WO2002074795A2 - Oligomeric complexes of chimeric proteins with enhanced immunogenic potential - Google Patents
Oligomeric complexes of chimeric proteins with enhanced immunogenic potential Download PDFInfo
- Publication number
- WO2002074795A2 WO2002074795A2 PCT/EP2002/000628 EP0200628W WO02074795A2 WO 2002074795 A2 WO2002074795 A2 WO 2002074795A2 EP 0200628 W EP0200628 W EP 0200628W WO 02074795 A2 WO02074795 A2 WO 02074795A2
- Authority
- WO
- WIPO (PCT)
- Prior art keywords
- influenza
- recombinant
- antigen
- vaccine
- protein
- Prior art date
- Legal status (The legal status is an assumption and is not a legal conclusion. Google has not performed a legal analysis and makes no representation as to the accuracy of the status listed.)
- Ceased
Links
Classifications
-
- C—CHEMISTRY; METALLURGY
- C07—ORGANIC CHEMISTRY
- C07K—PEPTIDES
- C07K14/00—Peptides having more than 20 amino acids; Gastrins; Somatostatins; Melanotropins; Derivatives thereof
- C07K14/005—Peptides having more than 20 amino acids; Gastrins; Somatostatins; Melanotropins; Derivatives thereof from viruses
-
- A—HUMAN NECESSITIES
- A61—MEDICAL OR VETERINARY SCIENCE; HYGIENE
- A61P—SPECIFIC THERAPEUTIC ACTIVITY OF CHEMICAL COMPOUNDS OR MEDICINAL PREPARATIONS
- A61P31/00—Antiinfectives, i.e. antibiotics, antiseptics, chemotherapeutics
- A61P31/12—Antivirals
- A61P31/14—Antivirals for RNA viruses
- A61P31/16—Antivirals for RNA viruses for influenza or rhinoviruses
-
- A—HUMAN NECESSITIES
- A61—MEDICAL OR VETERINARY SCIENCE; HYGIENE
- A61K—PREPARATIONS FOR MEDICAL, DENTAL OR TOILETRY PURPOSES
- A61K39/00—Medicinal preparations containing antigens or antibodies
-
- C—CHEMISTRY; METALLURGY
- C07—ORGANIC CHEMISTRY
- C07K—PEPTIDES
- C07K2319/00—Fusion polypeptide
- C07K2319/40—Fusion polypeptide containing a tag for immunodetection, or an epitope for immunisation
-
- C—CHEMISTRY; METALLURGY
- C07—ORGANIC CHEMISTRY
- C07K—PEPTIDES
- C07K2319/00—Fusion polypeptide
- C07K2319/70—Fusion polypeptide containing domain for protein-protein interaction
-
- C—CHEMISTRY; METALLURGY
- C07—ORGANIC CHEMISTRY
- C07K—PEPTIDES
- C07K2319/00—Fusion polypeptide
- C07K2319/70—Fusion polypeptide containing domain for protein-protein interaction
- C07K2319/73—Fusion polypeptide containing domain for protein-protein interaction containing coiled-coiled motif (leucine zippers)
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N2760/00—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA ssRNA viruses negative-sense
- C12N2760/00011—Details
- C12N2760/16011—Orthomyxoviridae
- C12N2760/16111—Influenzavirus A, i.e. influenza A virus
- C12N2760/16122—New viral proteins or individual genes, new structural or functional aspects of known viral proteins or genes
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N2760/00—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA ssRNA viruses negative-sense
- C12N2760/00011—Details
- C12N2760/16011—Orthomyxoviridae
- C12N2760/16211—Influenzavirus B, i.e. influenza B virus
- C12N2760/16222—New viral proteins or individual genes, new structural or functional aspects of known viral proteins or genes
Definitions
- the present invention relates to a chimeric protein comprising an antigen and an oligomerisation domain.
- the present invention relates further to recombinant oligomeric protein complexes comprising said chimeric protein and the use thereof for the manufacture of a vaccine.
- Hsp16.3 of Mycobacterium tuberculosis and several bacterial toxins Hsp16.3, an immunodominant antigen of Mycobacterium tuberculosis with serodiagnostic value, occurs as an oligomeric structure, presumably based on trimers (Chang et al., 1996).
- Cholera toxin as well as the closely related heat-labile toxin from Esche ⁇ chia coli is composed of two subunits, A and B, which form an oligomeric assembly AB 5 .
- the B subunit portion of cholera toxin can be used as an immunizing agent in humans, providing protection against both cholera and diarrhoea caused by enterotoxigenic E. coli (Sanchez et al. 1990).
- B oligomer which is a constituent of pertussis toxin, can be used to elicit immunoprotective responses against Bordetella pertussis. Also viral antigens occur often as oligomeric structures.
- herpes simplex virus type 1 glycoprotein B (Lin et al., 1996) or the flavivirus non-structural protein NS1 , which has been used in a recombinant vaccine against dengue-2 and which exists normally as a homodimer in infected cells (Winkler et al., 1988).
- the HIV-1 envelope molecules gp41 and gp120 which may be interesting targets for vaccine development, likewise form an oligomeric structure (Burton, 1997).
- the predominant antigens of influenza virus are also oligomers. Haemagglutinin (HA) occurs naturally as a homotrimer.
- NA Neuraminidase
- oligomeric antigens are presumed to keep their oligomeric structure in these vaccines, this is not always the case.
- the oligomeric antigens may lose their oligomeric structure during the viral disruption step.
- influenza viruses there is an additional complication due to the fact that they undergo significant antigenic variation in their two surface antigens haemagglutinin (HA) and neuraminidase (NA) (antigenic drift).
- influenza vaccine Due to the variability of these two proteins a broad spectrum, long lasting vaccine against influenza has so far not been developed.
- the influenza vaccine commonly used has to be adapted almost every year to follow the antigenic drift. When more drastic changes occur in the virus, known as antigenic shift, a previous vaccine is no longer protective.
- the present vaccines are based on virus material that has been produced in chicken eggs. Although these vaccine preparations have been found to be effective against an influenza infection caused by the homologous virus strain, there are several drawbacks, such as the production time, which makes it impossible to put an adapted vaccine on the market on short term notice.
- Recombinant vaccines can be based on selected epitopes and are generally safer and cheaper to produce.
- the antigen can be fused to immunostimulatory domains to avoid or limit the use of adjuvant in the vaccine preparation, or to boost the immune response of weakly immunogenic epitopes.
- Recombinant vaccines have been developed against several major diseases, such as measles, tetanus, pertussis, TBC, hepatitis B, cholera and influenza.
- Several others such as e.g. a recombinant vaccine against HIV, are under development.
- recombinant vaccines against influenza virus have been described in WO9406468, WO9407533, W09518861 and WO9520660.
- a recombinant vaccine based on the membrane protein M2 has been developed, which has the additional advantage to induce a broad spectrum, long-term protection (Neirynck et al., 1999; WO9303173, WO9907839, W09928478).
- NA Laver and Valentine, 1969; Bucher and Kilboume, 1972; Varghese et al., 1983; Ward et al., 1983
- M2 Sudgrue and Hay, 1991
- recombinant preparations of NA only partly yield homotetramers, the major part of the preparation being monomers and dimers.
- antigenic epitopes are as well, if not better accessible in these mono- and dimers, surprisingly, we found that tetrameric molecules were considerably superior in eliciting a specific antibody response.
- tetrameric preparations of these molecules can be obtained by an additional purification step of the recombinant protein, such as size exclusion chromatography, such purification would lead to an important loss in yield. Furthermore, renewed dissociation of the purified material cannot be excluded.
- a spontaneous tetramerisation could be obtained of the fusion protein, yielding a recombinant protein in an almost purely tetrameric form.
- these fusion tetramers showed a similar enhanced antigenic capacity as the purified tetrameric, recombinant protein. It is the object of the invention to provide a highly immunogenic recombinant antigen protein complex, preferably a recombinant influenza antigen protein complex.
- Said oligomerisation domain is heterologous, i.e. it is derived from another protein than the antigen.
- the oligomerisation domain is driving the oligomerisation of the chimeric protein to form a recombinant oligomeric protein complex.
- the degree of oligomerisation (dimeric, trimeric, tetrameric or higher) of the chimeric protein is identical to the degree of oligomerisation of the naturally occurring protein complex from which the antigen is derived and the antigenic domain of the chimeric protein is presented in a tertiary structure that is similar or identical to that of the tertiary structure of the antigenic domain in the naturally occurring protein.
- said antigen is an influenza antigen. More preferably, said antigen is influenza neuraminidase or influenza M2-protein or a functional fragment thereof. Most preferably, said antigen is chosen from the group consisting of influenza A neuraminidase, influenza A M2 or influenza B NB-protein.
- Oligomerisation domains are known to the people skilled in the art and have, amongst others, been described in W09637621 , W09818943, WO9856906, W09962953 and WO0069907.
- the oligomerisation domain is a leucine zipper. More preferentially, the oligomerisation domain is a leucine zipper derived from the yeast transcription factor GCN4, or a modified form thereof. Most preferentially, the oligomerisation domain is a modified leucine zipper, derived from the yeast transcription factor GCN4, as described by Harbury et al. (1993).
- a preferred embodiment of the invention is the influenza B neuraminidase or a functional fragment thereof such as the neuraminidase B ecto-domain, fused to an oligomerisation domain such as a modified leucine zipper, derived from the yeast transcription factor GCN4, as described by Harbury et al. (1993).
- Another preferred embodiment is the influenza B NB-protein, or a functional fragment thereof, fused to an oligomerisation domain. It is an aim of the present invention to present the recombinant protein complex in a conformation that resembles the conformation of the naturally occurring protein complex. In cases where the naturally occurring protein complex has a defined enzymatic activity, as is the case for influenza neuraminidase, the recombinant protein complex will have a comparable enzymatic activity.
- the chimeric protein may comprise other polypeptide sequences, such as linker sequences or polypeptide sequences that enhance the immune response.
- polypeptide sequences that enhance the immune response are known to the person, skilled in the art and include, as a non-limiting example, one or more copies of the third complement protein fragment d (C3d; Dempsey et al., 1996) or tetanus toxin fragment C, or Escherichia coli enterotoxin fragment A or B, or T-cell epitopes derived from the same pathogen as the antigen.
- Another aspect of the invention is a recombinant oligomeric protein complex comprising a chimeric protein according to the invention.
- said recombinant oligomeric protein complex is a dimer, or a tetramer. More preferentially, said recombinant oligomeric protein complex is a homodimer or a homotetramer.
- said oligomeric protein complex elicits a higher immune response than the monomeric subunit.
- a preferred embodiment of the invention is a recombinant oligomeric protein complex that has a comparable enzymatic activity as the naturally occurring oligomeric protein complex of which the antigen, comprised in the chimeric protein that forms said recombinant oligomeric protein complex, is derived.
- Still another aspect of the invention is a nucleic acid, encoding a chimeric protein according to the invention.
- a preferred embodiment is a nucleic acid, comprising the sequence presented in SEQ ID N° 1.
- Another preferred embodiment is a nucleic acid, comprising the sequence presented in SEQ ID N° 3.
- Still another preferred embodiment is a nucleic acid comprising the sequence presented in SEQ ID N° 5.
- a special embodiment is a nucleic acid, according to the invention that may be used in DNA vaccination.
- Vectors for DNA vaccination are known to the person skilled in the art and are described, amongst others, in WO9604394, W09728259 and WO9908713. Methods for DNA vaccination have been described amongst others in WO0012121.
- a further aspect of the invention is an expression vector comprising a nucleic acid according to the invention and allowing the expression of a chimeric protein, according to the invention.
- Said expression vector can be any eukaryotic or prokaryotic expression vector, as known to the person skilled in the art.
- the expression vector is pACGCN4NAs (Deposition at BCCM - (deposit nr LMBP 4270)), comprising the antigenic head domain of NA wherein the N-terminal part has been replaced by a modified leucine zipper derived from the yeast transcription factor GCN4, which is imposing tetramerisation (Harbury et al., 1993).
- This construct is fused to the secretion signal of influenza haemagglutinin and the construct is placed under control of the baculovirus polyhedrin promoter.
- Another preferred embodiment is pACsM2eGCN4 (deposit nr LMBP 4271), comprising the ectodomain of M2, fused at its N-terminus to the GP67 secretion signal of Baculovirus and at its C-terminus to the tetramerising, modified leucine zipper derived from the yeast transcription factor GCN4 (Harbury et al., 1993).
- Still another preferred embodiment is pACsM2eGCN4C3d (Deposition at BCCM - (deposit nr LMBP 4463)), where said ectodomain of M2, placed after the GP67 secretion signal of Baculovirus and fused to the GCN4 leucine zipper, is fused to the C3d domain.
- Still another aspect of the invention is a host cell, transformed with an expression vector according to the invention. Said cell can be any prokaryotic or eukaryotic host cell. Transformation procedures are known to the person skilled in the art.
- a further aspect of the invention is the use of a chimeric protein according to the invention and/or the use of a recombinant oligomeric protein complex according to the invention for the preparation of a vaccine against influenza.
- a special embodiment is the use of said chimeric protein whereby said chimeric protein comprises SEQ ID N° 2, SEQ ID N° 4 or SEQ ID N° 6.
- the chimeric protein may also be used to elicit monoclonal or polyclonal antibodies, using techniques known to the person skilled in the art, whereby said antibodies can be used for diagnostic or therapeutic purposes. Human or humanised antibodies may be especially useful as therapeutics for people with a decreased immune response, such as HIV patients.
- Still another aspect of the invention is a vaccine against influenza, comprising a chimeric protein and/or a recombinant oligomeric protein complex according to the invention.
- Still another aspect of the invention is a vaccine against influenza, comprising a substantially pure tetrameric form of a recombinant influenza antigen.
- said recombinant influenza antigen is recombinant influenza neuraminidase, or a functional fragment thereof.
- said recombinant influenza antigen is recombinant M2, or a functional fragment thereof.
- said influenza vaccine is fused to a heterologous oligomerisation domain, most preferably, said influenza vaccine is fused to the tetramerising, modified leucine zipper derived from the yeast transcription factor GCN4 (Harbury et al., 1993).
- a preferred embodiment is a vaccine, comprising a substantially pure tetrameric form of neuraminidase or a functional fragment thereof, whereby said substantially pure tetrameric form has an enzymatic activity that is comparable to naturally occurring influenza neuraminidase.
- Still another aspect of the invention is the use of chimeric protein according to the invention and/or the use of a recombinant oligomeric protein complex according to the invention to screen inhibitors of the biological activity of the naturally occurring protein complex.
- a preferred embodiment is said use to screen inhibitors of influenza A or influenza B neuraminidase, or inhibitors of influenza A M2 or influenza B NB-protein.
- - Chimeric protein as used here means that the protein is composed of at least two poiypeptides, which do not occur in the same protein in the natural form
- - Antigen as used here means an antigen, derived from a naturally occurring oligomeric protein from a pathogenic organism or micro-organism, including viruses, and can be used in a host, preferably, but not limited to a human host, to elicit an immune response against said pathogenic organism or micro-organism.
- - Recombinant oligomeric protein complex is a protein complex wherein at least one of the subunits is a chimeric protein comprising an oligomerisation domain.
- - Recombinant antigen as used here means that said antigen is produced by recombinant DNA techniques.
- the antigen may be produced in any prokaryotic or eukaryotic host cell, such as, as a non-limiting example, Escherichia coli, Bacillus subtilis, yeast such as Saccharomyces cerevisiae or Kluyveromyces sp., fungal cells, insect cells, plant cells or mammalian cells.
- Comparable enzymatic activity means that both the naturally occurring protein complex and the recombinant oligomeric protein complex can perform at least one identical biochemical transformation of at least one substrate, but that the specific activity of the enzymatic complexes may differ.
- Identical biochemical transformation means that the substrate by the action of the enzymatic activity is transformed in an identical end product or identical end products.
- Substantially pure tetrameric form of a recombinant antigen means that said recombinant antigen is at least for 80%, preferably at least for 90% in the tetrameric form.
- - Functional fragment of influenza neuraminidase or of influenza M2 is any fragment that can elicit an immune response against influenza virus.
- a functional fragment of influenza M2 is the M2 ecto-domain.
- vaccine as used here can be any protein based vaccine, including injectable as well as mucosal vaccines.
- GCN4 modified GCN4 leucine zipper
- Figure 2 Construction of pACsM2eGCN4
- Phprom polyhedrin promoter sGP67 : secretion signal of the baculovirus GP67 protein
- M2e extracellular part of M2 (M2 ectodomain)
- GCN4 modified GCN4 leucine zipper bla : ⁇ -lactamase ori : origin of replication bold grey line : baculovirus homology region
- Figure 3 Flow diagram for the construction of pACsM2eGCN4C3d. Only restriction sites relevant to the cloning procedure have been indicated.
- Figure 4 Antibody response against different oligomeric subforms of recombinant neuraminidase.
- Figure 5 Survival of mice vaccinated with different oligomeric subforms of recombinant neuraminidase after a lethal challenge with homologous, mouse-adapted influenza virus.
- Figure 6 Analysis of GCN4NAs expression by Western blot.
- Figure 7 Sucrose gradient pattern of secreted neuraminidase and secreted chimeric GCN4NAS.
- Figure 8 Proposed structure of GCN4NAs based on the known structure of its two constituent domains.
- GCN4NAs is a tetramer as shown by chemical cross-linking of its subunits.
- Lane 1 30 min incubation of GCN4NAs with 1.2 mM BS3
- Lane 2 5 min incubation of GCN4NAs with 1.2 mM BS3
- Lane 3 30 min incubation of GCN4NAs with 0.6 mM BS3 Lane 4; 5 min incubation of GCN4NAs with 0.6 mM BS3 Lane 5: 30 min incubation of GCN4NAs with 0.3 mM BS3 Lane 6: 5 min incubation of GCN4NAs with 0.3 mM BS3 Lane 7: GCN4NAs without cross-linker
- Lane 8 MW Figure 10: Characterisation of sM2eGCN4 expression.
- FIG 11 Analysis by 12 % SDS-PAGE of proteins secreted by baculovirus-infected Sf9 cells in TC100 medium. TCA precipitated proteins from 800 ⁇ l medium were dissolved in loading buffer.
- Lanes A1 and B1 were loaded with proteins derived from cells infected with baculovirus obtained by recombination with an empty expression vector. Lanes A2 and B2 were loaded with proteins derived from cells infected with baculovirus containing the genetic information for expression of sM2eGCN4C3d.
- mice were injected i.p. either with PBS + adjuvant or sM2eGCN4C3d + adjuvant, and the injections were repeated twice at 2 weeks interval (cf. Example 13). Serum was taken 10 days after each injection, and antibody titers were determined using either M2e-peptide or sM2eGCN4C3d for trapping.
- Vac, b1 and b2 serum taken after first injection, first boost and second boost, respectively.
- mice were immunized three times with PBS or 10 ⁇ g sM2eGCN4C3d (cf.
- Example 13 Example 13
- Example 13 challenged with homologous, mouse-adapted X47 virus Examples
- the baculovirus transfer vector pAC2IVNAs (containing the cDNA sequence of the N2 neuraminidase of A/Victoria/3/75 influenza virus of which the membrane anchor was substituted by the cleavable signal sequence of the haemagglutinin; described in detail in Deroo et al., 1996) was used as a template to generate two PCR products using the primer pairs BACfor/GCN4nh (denaturation: 94°C, 1 min; annealing 57°C, 1 min; synthesis 75°C, 30 sec) and GCN4cooh/BACrev (denaturation: 94°C, 1 min; annealing 59°C, 1 min; synthesis 75°C, 2 min 30 sec), which were subsequently digested with Pstl/Hindlll and Bcll/Xbal, respectively.
- the resulting fragments and a 5' end kinated synthetic DNA fragment (GCN4pos/GCN4neg complementary oligonucleotide pair) were then ligated with the Pstl/Xbal 10089 bp vector fragment of pAC2IVNAs.
- the inserted sequence in the baculovirus transfer vector obtained in this way (pACGCN4NAs), codes for the antigenic and catalytic head domain of the neuraminidase (NA) preceded by a modified GCN4 leucine zipper which promotes the formation of a tetrameric protein (Harbury et al., 1993), and by the secretion signal of the influenza haemagglutinin (sHA).
- baculovirus polyhedrin promotor Phprom
- the corresponding recombinant baculovirus designated AcNPV[GCN4NAs]
- the construction is summarized in Fig. 1.
- the GP67 secretion signal was fused with the M2e fragment (coding for the ectodomain of the M2 protein) obtained by PCR amplification (primers M2Ss and UM2ECa; denaturation: 94°C, 1 min; annealing: 62°C, 1 min; synthesis: 75°C, 20 sec) and subsequent treatment with HindUl.
- This construct referred to as pUCsgpM2e, was used as a template to generate a new PCR fragment (primers GP67s and M2rev; denaturation: 94°C, 1 min; annealing 56°C, 1 min; synthesis 75°C, 30 sec), which was digested with Spel and BspEI.
- the GCN4 PCR fragment obtained from pACGCN4NAs (primers GCNfor and GCNrev; denaturation: 94°C, 1 min; annealing 58°C, 1 min; synthesis 75°C, 30 sec) was then ligated with the former fragment together with the Spel/Bglll 9610 bp vector fragment of pACGP67A.
- the sequence coding for the M2 ectodomain (M2e) is fused at its C-terminus to a modified GCN4 leucine zipper which is able to induce tetramerization (Harbury et al., 1993), and is preceded by the GP67 secretion signal (sGP67), and by the polyhedrin promoter (Phprom).
- the corresponding recombinant baculovirus (designated AcNPV[sM2eGCN4]) was generated by calcium phosphate cotransfection of Sf9 insect cells with BaculoGold baculovirus DNA (Pharmingen, San Diego, CA. , USA), following the procedure as described in King and Possee (1992). The construction is summarized in Fig. 2.
- Example 3 Construction of pACsM2eGCN4C3d
- the plasmid pSG5.C3d3.YL was a kind gift from Dr. D.T. Fearon, Department of Medicine, University of Cambridge School of Medicine, Cambridge, UK.
- the C3d genetic information was first amplified and subcloned in the vector pUC18 (Norrander et al.,1983) as follows:
- the C3d sequence was PCR amplified (primers C3ds and C3da, pSG5.C3d3.YL as template; denaturation: 94 °C, 30 sec; annealing: 60°C, 20 sec; synthesis: 72°C, 2 min), followed by cleavage with Spel and Bglll to allow insertion into Spel/Bglll digested, intermediate vector pUC18f.
- the latter had been created by inserting a Spel restriction site in Smal opened pUC18, using the adaptor 5TCACTAGTGA3', and by inserting a Bglll restriction site in the Hindll opened vector, using the adaptor 5'CAGATCTG3'.
- the result of cloning the PCR fragment in pUC18f was the plasmid pUCC3d.
- the starting plasmid pSG5.C3d3.YL was cleaved also with Xbal, followed by blunting with T4 DNA polymerase, and by subsequent digestion with BspEI, which provided a 680 bp fragment.
- the sM2eGCN4 coding sequence was PCR amplified (denaturation: 94 °C, 1 min; annealing: 57°C, 1 min; synthesis: 75°C, 30 sec), and then treated with Spel and BamHl.
- the resulting fragment was inserted into Spel/BamHI digested pACGP67A (baculovirus transfer vector purchased from Pharmingen, San Diego, CA., USA). This provided the intermediate construct pACsM2eGCN4f.
- the aforementioned plasmid pUCC3dEEF was digested with Bglll and EcoRI to provide a 1094 bp fragment coding for C3dEEF, which was subcloned in BamHl and EcoRI opened pACsM2eGCN4f. This provided the plasmid pACsM2eGCN4C3d.
- the polyhedrin promotor (Phprom) is followed by a multi-component fusion gene coding for the GP67 secretion signal (sGP67), the M2e ectodomain (M2e), the GCN4 leucine zipper, the mouse C3d domain and a C-terminal ⁇ EF' tag.
- the corresponding baculovirus (designated AcNPV[sM2eGCN4C3d]) was generated by calcium phosphate cotransfection of Sf9 insect cells with BaculoGold baculovirus DNA (Pharmingen, San Diego, CA., USA), following the procedure as described in King and Possee (1992). The construction is summarized in Fig. 3.
- Example 4 Analysis of antibody response against different oligomeric subforms of purified secreted neuraminidase
- NAs Secreted recombinant NA
- a baculovirus expression system was produced by a baculovirus expression system and subsequently purified according to Deroo et al. (1996).
- Superdex 200 gel filtration which is the final step of the purification procedure described in Deroo et al. (1996), the fractions corresponding to monomeric, dimeric and tetrameric NAs were pooled separately, and concentrated by ultrafiltration using Centriplus devices (10 kDa cut-off) (Am icon, Danvers, MA., USA).
- mice Groups of 12 female Balb/c mice (SCK Mol, Belgium) were then immunized three times by subcutaneous injection with 1 ⁇ g of a specific oligomeric subform in the presence of a low-reactogenic adjuvant, as described in Deroo et al. (1996). Two weeks after each immunization, blood was collected from the tail vein and serum was prepared. Serum samples were subsequently analyzed by ELISA. For this purpose, 96-well plates were coated with purified, pronase-cleaved NA (Deroo et al., 1993), and incubated with 2-fold serum dilutions.
- Serum antibody titers were measured by adding alkaline phosphatase conjugated goat anti-[mouse IgG] antibody (Sigma Chemical Co., St. Louis, MO., USA) and p-nitrophenyl phosphate (Sigma Chemical Co., St. Louis, MO., USA) as a substrate.
- the serum antibody titer corresponds to the log 2 value of the dilution factor which gave an OD of 0.5 above the control.
- Mice immunized with tetrameric NAs show a superior antibody respons throughout the immunization regimen (Fig. 4).
- Example 5 Survival of mice challenged with a lethal dose of influenza virus after vaccination with different oligomeric subforms of purified, secreted neuraminidase Groups of 12 female Balb/c mice were immunized subcutaneously with different oligomeric subforms of purified, secreted neuraminidase (NAs), as outlined under example 4. Three weeks after the third injection, mice were challenged with a potentially lethal dose of mouse-adapted influenza virus (X47 reassortant strain) as described in Deroo et al. (1996). No lethality was observed among the animals that received tetrameric NAs vaccine. By contrast, only 75% and 50% of the animals immunized with dimeric and monomeric NAs, respectively, survived the challenge (Fig. 5).
- Example 6 Analysis of GCN4NAs expression by Western blotting
- Log-phase Sf9 insect cells were inoculated with the indicated baculovirus at high multiplicity of infection (>10). Cells were subsequently transferred to serum-free TC100 medium (Gibco BRL, Bethesda, MD., USA) and further incubated for 48 h before harvesting the supernatant. Proteins were precipitated by adding an equal volume of acetone (pre-equilibrated at -20°C) and subsequently analysed by 12% reducing SDS-PAGE followed by Western blotting.
- NAs secreted neuraminidase
- GCN4NAs secreted GCN4-fused neuraminidase
- ELISA was carried out in 96-well plates coated with a rabbit IgG fraction raised against purified, pronase-cleaved neuraminidase (cf. example 6). Gradient fractions were added to the plates, and bound NAs was detected by addition of biotin-conjugated, anti-pronase- cleaved NA rabbit IgG. Plates were developed by incubating them with streptavidin - alkaline phophatase conjugate (Gibco BRL, Bethesda, MD., USA) and p-nitrophenyl phosphate as a substrate. OD values were read at 405 nm. Analysis of enzymatic activity was performed as described in Deroo et al.
- Cross-linkers were obtained from Pierce (Rockford, IL, USA).
- NC membranes Electroblotting from SDS PAGE gels onto nitrocellulose (NC) membranes was performed using a Mini Trans-Blot cell (BioRad, Hercules, CA, USA) and required 45 min at 100 V. Thereafter, NC membranes were blocked in PBS containing 2% BSA for 2h. Blots were incubated with anti-NA rabbit serum (cf. example 6) diluted (1/5000) in PBS containing 1 % BSA and 0.1% Tween- 20 (PBT). After washing away unbound antibodies, alkaline phosphatase conjugated goat anti-rabbit-lgG serum (Organon Teknika, West Chester, PA, USA) was added at a dilution of 1/7000 in PBT.
- anti-NA rabbit serum cf. example 6
- PBT Tween- 20
- Log-phase Sf9 insect cells were inoculated with baculovirus AcNPV[sM2eGCN4] (example 2) or control virus at high multiplicity of infection (>10). Cells were subsequently transferred to serum-free TC100 medium (Gibco BRL, Bethesda, MD., USA) and further incubated for 48 h before harvesting the supernatant. Proteins were precipitated by adding an equal volume of acetone (pre-equilibrated at -20°C), dissolved in loading buffer and separated by 15% reducing SDS-PAGE, followed by Western blotting. Bands were visualized using the monoclonal antibody 2C9 directed against the M2e domain (Neirynck et al.
- Example 10 Characterisation of sM2eGCN4C3d expression
- Log-phase Sf9 insect cells were inoculated with baculovirus AcNPV[sM2eGCN4C3d] (cf. example 3) or control virus ("mock infection") at high multiplicity of infection (>10).
- Cells were subsequently transferred to serum-free TC100 medium (Gibco BRL, Bethesda, MD., USA) and further incubated for 48 h before harvesting the supernatant. Proteins were analyzed by precipitation with ice-cooled TCA and subsequently separated by 12 % reducing SDS-PAGE, followed by SyproOrange staining (Molecular Probes, Eugene, OR., USA).
- sM2eGCN4C3d was revealed as a band of ⁇ 41 kDa, which was not present in the medium of 'mock' infected Sf9 cells (Fig. 11).
- baculovirus has been generated by calcium phosphate cotransfection of Sf9 cells with transfer vector pACGP67A without an insert for expression, and BaculoGold baculovirus DNA (Pharmingen, San Diego, CA., USA), following the procedure as described in King and Possee (1992).
- sM2eGCN4C3d was again visualized as a band of ⁇ 41 kDa using the anti-M2e monoclonal antibody 2C9 (Neirynck et al., 1999), followed by incubation with a secondary antibody (rat anti-[mouse IgG] - peroxidase conjugate; Sigma Chemical Co., St. Louis, MO., USA) and 'Renaissance' chemiluminescent substrate solution (NEN Life Science Products, Boston, MA., USA).
- rat monoclonal antibody YL 1/2 against the 'EEF'tag (Abeam Ltd, Cambridge, UK) was used, or sheep polyclonal antibody against mouse complement 3 (Biogenesis, Poole, UK).
- the following secondary antibodies were used: mouse monoclonal anti-rat kappa and lambda light chains (clones RT-39 & RL-6) conjugated with alkaline phosphatase, and donkey anti-sheep IgG conjugated with alkaline phosphatase, respectively (Sigma, St. Louis, MO., USA).
- the blotted proteins were stained with amido black, the -41 kDa band was isolated by cutting the membrane, and N-terminal sequence analysis was carried out according to Bauw et al. (1987). The first four amino acids were identified as serine, leucine, leucine and threonine, respectively. This result demonstrates that cleavage of the GP67 signal sequence has been executed correctly, and confirms that the ⁇ 41 kDa band is without doubt sM2eGCN4C3d.
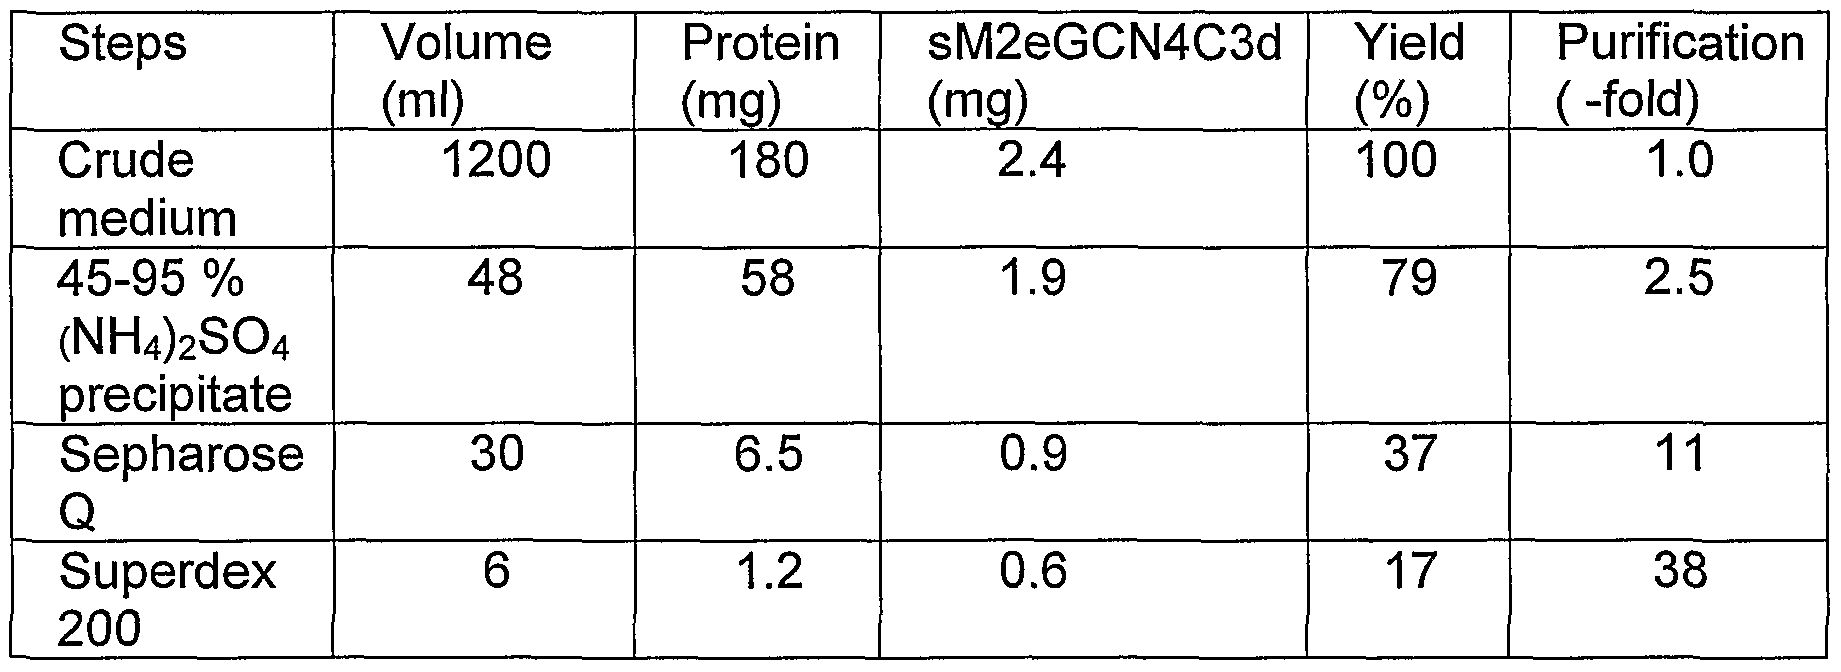
- the pellet was redisolved in 50 mM Tris.CI buffer, pH 7.2, (approximately 1/20th of the original volume of the medium), and desalted over a HiPrep Sephadex G25 column (Amersham Pharmacia Biotech, Uppsala, Sweden) equilibrated in 50 mM Tris.CI, pH 7.2.
- the desalted protein solution was loaded on a Q-Sepharose FF column (h: 9 cm, d: 1.5 cm; Amersham Pharmacia Biotech, Uppsala, Sweden) equilibrated in 50 mM Tris buffer, pH 7.2, and elution was by a salt gradient of 200 to 400 mM NaCl in 20 mM Tris buffer, pH 7.2.
- This Superdex 200 column had previously been calibrated using a mixture of highly purified proteins (HMW and LMW calibration kits (Amersham Pharmacia Biotech, Uppsala, Sweden). As shown in Fig. 12, sM2eGCN4C3d was detected only in fractions nearly coinciding with those of aldolase (theoretical molecular mass 179 kDa), as can be expected for tetrameric sM2eGCN4C3d.
- Example 12 Characterization of the oligomeric status of sM2eGCN4C3d by cross-linking.
- Samples (10 ⁇ l) of partially purified sM2eGCN4C3d (approx. 0.5 ⁇ g, in PBS; cf. example 11) were incubated with cross-linker BS3 (Pierce, Rockford, IL, USA) at final concentrations of 4 to 12 mM.
- the cross-linker was added from a freshly made 40 mM stock solution in DMSO. The reactions were incubated for 10 minutes at room temperature, and quenched for 15 minutes by addition of 1 M Tris buffer, pH 7.5, to a final concentration of 300 mM.
- SDS-PAGE analysis was carried out on a MiniProtean II apparatus (BioRad, Hercules, CA, USA) using 4-15 % precast gradient gels. Electroblotting from SDS-PAGE gels onto nitrocellulose (NC) membranes was performed using a Mini Trans-Blot cell (BioRad, Hercules, CA, USA) and required 1 hour at 100 V.
- NC membranes were blocked overnight at 4 °C in PBS containing 2 % BSA. Blots were incubated with anti-M2e monoclonal antibody 2C9 in TBS-T (50 mM Tris buffer, pH 7.0, 50 mM NaCl, and 0.1 % Tween- 20). After washing away unbound antibodies, the blot was screened with secondary antibody (rat anti-[mouse IgG] - peroxidase conjugate; Sigma chemical Co., St. Louis, MO., USA) and positive signals were revealed after addition of 'Renaissance' chemiluminescent substrate solution (NEN Life Science Products, Boston, MA., USA).
- secondary antibody rat anti-[mouse IgG] - peroxidase conjugate
- Prestained broad range molecular weight marker proteins (BioRad, Hercules, CA, USA) were used as references.
- treatment of sM2eGCN4C3d with the cross-linker BS3 resulted in the formation of covalently linked oligomers.
- the major cross-linked species has an estimated molecular mass of approximately 164 kDa, while the monomer had a molecular mass of approximately 41 kDa. This result confirms data obtained by ultrafiltration and gelfiltration, which all indicate that sM2eGCN4C3d exists in solution as a tetramer.
- Example 13 Analysis of the in vivo antibody response against sM2eGCN4C3d
- sM2eGCN4C3d Secreted, recombinant sM2eGCN4C3d was produced by a baculovirus expression system and purified, as outlined in examples 10 and 11. Fractions containing recombinant protein were concentrated using Vivaspin-30 and Centricon-100 ultrafiltration devices (Millipore Corporation, Bedford, MA., USA).
- mice Groups of 7 female Balb/c mice (Charles River Laboratories, Sulzfeld Germany) at the age of 8 weeks were immunized by intraperitoneal injection with 10 ⁇ g sM2eGCN4C3d in the presence of Ribi adjuvant (25 ⁇ g monophosphoryl lipid A and 25 ⁇ g trehalose-6,6-dimycolate; cf. Neirynck et al., 1999) per mouse. Control mice received adjuvant dispersed in phosphate-buffered saline. The animals were housed in a temperature-controlled environment with 12 h light/dark cycles, and received food and water ad libitum.
- Ribi adjuvant 25 ⁇ g monophosphoryl lipid A and 25 ⁇ g trehalose-6,6-dimycolate; cf. Neirynck et al., 1999
- 96-well plates were coated overnight at 4°C with 50 ⁇ l of 10 ⁇ g/ml anti-mouse complement 3 polyclonal antibodies (ab3163, Biogenesis Ltd, Poole, UK) and blocked with 150 ⁇ l PBS containing 1 % BSA during 1 hour. With the latter coating, capturing of sM2eGCN4C3d from insect cell medium was allowed during 1 hour 30 minutes at room temperature. After washing, a series of 1/2 dilutions of the different serum samples, starting with a 1/50 dilution, were loaded on peptide- or sM2eGCN4C3d protein coated wells.
- Bound antibodies were detected with a peroxidase-labeled antibody directed against mouse lgG1 and lgG3 (Southern Biotechnology Associates, Inc.), respectively, diluted 1/6000 in PBS containing 1% BSA and 0.05% Tween-20. After washing, the microtiter plates were incubated for 20 minutes with 3,3',5,5'-tetramethylbenzidine liquid substrate for peroxidase (Sigma, St. Louis, MO., USA). The reaction was stopped by addition of 1 M H 3 P0 and the absorbance at 450 nm was measured.
- Example 14 Protection of mice challenged with a lethal dose of influenza virus after vaccination with sM2eGCN4C3d
- mice Groups of 7 female pathogen-free Balb/c mice (Charles River Laboratories Sulzfeld, Germany) were immunized intraperitoneal with sM2eGCN4C3d, as described in example 13. Two weeks after the last immunisation, the mice were challenged intranasally with 14 LD 5 o of mouse-adapted (m.a.) X47 (Neirynck et al., 1999). As presented in figure 15, sM2eGCN4C3d vaccinees were protected against a lethal dose of homologous m.a. influenza A virus.
- Table I PCR Primers and complementary oligonucleotide pair PCR primers
- UM2ECa 5' CGAAGCTTACTAGTTCACGGATCCCCACTTGAATCGTTGCATCTGCACCC
- the peak values of the enzymatic activity and the ELISA read-out obtained after sucrose gradient centrifugation were used to deduce a rough estimation of the relative specific activities.
- the specific enzymatic activity of GCN4NAs amounts to at least 70% of that of the tetrameric form of the unfused NAs protein.
- A2 (N2) neuraminidase of the X-7 influenza recombinant determination of molecular size and subunit composition of the active unit. J Virol, 10, 60 - 66.
Landscapes
- Health & Medical Sciences (AREA)
- Life Sciences & Earth Sciences (AREA)
- Chemical & Material Sciences (AREA)
- Virology (AREA)
- Organic Chemistry (AREA)
- Medicinal Chemistry (AREA)
- Molecular Biology (AREA)
- General Health & Medical Sciences (AREA)
- Gastroenterology & Hepatology (AREA)
- Biochemistry (AREA)
- Proteomics, Peptides & Aminoacids (AREA)
- Genetics & Genomics (AREA)
- Biophysics (AREA)
- Pharmacology & Pharmacy (AREA)
- Oncology (AREA)
- Communicable Diseases (AREA)
- Public Health (AREA)
- Veterinary Medicine (AREA)
- Pulmonology (AREA)
- General Chemical & Material Sciences (AREA)
- Animal Behavior & Ethology (AREA)
- Nuclear Medicine, Radiotherapy & Molecular Imaging (AREA)
- Chemical Kinetics & Catalysis (AREA)
- Medicines Containing Antibodies Or Antigens For Use As Internal Diagnostic Agents (AREA)
- Peptides Or Proteins (AREA)
- Medicines That Contain Protein Lipid Enzymes And Other Medicines (AREA)
- Preparation Of Compounds By Using Micro-Organisms (AREA)
Abstract
Description

Claims
Priority Applications (7)
| Application Number | Priority Date | Filing Date | Title |
|---|---|---|---|
| US10/466,655 US7449188B2 (en) | 2001-01-18 | 2002-01-18 | Recombinant oligometric protein complexes with enhanced immunogenic potential |
| AT02722030T ATE433491T1 (en) | 2001-01-18 | 2002-01-18 | OLIGOMERIC COMPLEXES OF CHIMERIC PROTEINS WITH ENHANCED IMMUNOGENIC POTENTIAL |
| DK02722030T DK1362109T3 (en) | 2001-01-18 | 2002-01-18 | Recombinant oligomeric protein complexes with enhanced immunogenic potential |
| AU2002252978A AU2002252978B9 (en) | 2001-01-18 | 2002-01-18 | Oligomeric complexes of chimeric proteins with enhanced immunogenic potential |
| EP02722030A EP1362109B1 (en) | 2001-01-18 | 2002-01-18 | Recombinant oligomeric protein complexes with enhanced immunogenic potential |
| DE60232577T DE60232577D1 (en) | 2001-01-18 | 2002-01-18 | OLIGOMERIC COMPLEXES OF CHIMERIC PROTEINS WITH IMPROVED IMMUNOGENIC POTENTIAL |
| CA2435000A CA2435000C (en) | 2001-01-18 | 2002-01-18 | Oligomeric complexes of chimeric proteins with enhanced immunogenic potential |
Applications Claiming Priority (2)
| Application Number | Priority Date | Filing Date | Title |
|---|---|---|---|
| EP01200193 | 2001-01-18 | ||
| EP01200193.9 | 2001-01-18 |
Publications (2)
| Publication Number | Publication Date |
|---|---|
| WO2002074795A2 true WO2002074795A2 (en) | 2002-09-26 |
| WO2002074795A3 WO2002074795A3 (en) | 2003-09-04 |
Family
ID=8179773
Family Applications (1)
| Application Number | Title | Priority Date | Filing Date |
|---|---|---|---|
| PCT/EP2002/000628 Ceased WO2002074795A2 (en) | 2001-01-18 | 2002-01-18 | Oligomeric complexes of chimeric proteins with enhanced immunogenic potential |
Country Status (9)
| Country | Link |
|---|---|
| US (1) | US7449188B2 (en) |
| EP (1) | EP1362109B1 (en) |
| AT (1) | ATE433491T1 (en) |
| AU (1) | AU2002252978B9 (en) |
| CA (1) | CA2435000C (en) |
| DE (1) | DE60232577D1 (en) |
| DK (1) | DK1362109T3 (en) |
| ES (1) | ES2327719T3 (en) |
| WO (1) | WO2002074795A2 (en) |
Cited By (24)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| WO2009133463A1 (en) * | 2008-04-30 | 2009-11-05 | University Of Copenhagen | Soluble influenza vaccine |
| WO2010003235A1 (en) * | 2008-07-08 | 2010-01-14 | Medicago Inc. | Soluble recombinant influenza antigens |
| WO2011126370A1 (en) * | 2010-04-09 | 2011-10-13 | Universiteit Utrecht Holding B.V. | Recombinant multimeric influenza proteins |
| WO2012011868A1 (en) * | 2010-07-23 | 2012-01-26 | Osterhaus A D M E | Influenza vaccine |
| WO2012128628A1 (en) * | 2011-03-22 | 2012-09-27 | Mucosis B.V. | Immunogenic compositions in particulate form and methods for producing the same |
| US8734778B2 (en) | 2002-12-16 | 2014-05-27 | Globeimmune, Inc. | Yeast-based vaccines as immunotherapy |
| US8865182B2 (en) | 2009-07-31 | 2014-10-21 | Paxvax, Inc. | Adenoviral-based vectors |
| US9452210B2 (en) | 2007-07-13 | 2016-09-27 | Medicago Inc. | Influenza virus-like particles (VLPS) comprising hemagglutinin produced within a plant |
| US9458470B2 (en) | 2007-11-27 | 2016-10-04 | Medicago Inc. | Recombinant influenza virus-like particles (VLPs) produced in transgenic plants expressing hemagglutinin |
| US9815873B2 (en) | 2011-03-23 | 2017-11-14 | Medicago Inc. | Method for recovering plant-derived proteins |
| US10272148B2 (en) | 2009-06-24 | 2019-04-30 | Medicago Inc. | Chimeric influenza virus-like particles comprising hemagglutinin |
| WO2021150874A1 (en) * | 2020-01-24 | 2021-07-29 | Wisconsin Alumni Research Foundation (Warf) | Recombinant influenza viruses with stabilized na |
| US11802273B2 (en) | 2014-06-20 | 2023-10-31 | Wisconsin Alumni Research Foundation (Warf) | Mutations that confer genetic stability to additional genes in influenza viruses |
| US11807872B2 (en) | 2019-08-27 | 2023-11-07 | Wisconsin Alumni Research Foundation (Warf) | Recombinant influenza viruses with stabilized HA for replication in eggs |
| US11826419B2 (en) | 2009-09-22 | 2023-11-28 | Medicago Inc. | Method of preparing plant-derived VLPs |
| US11851648B2 (en) | 2019-02-08 | 2023-12-26 | Wisconsin Alumni Research Foundation (Warf) | Humanized cell line |
| US12076387B2 (en) | 2010-03-23 | 2024-09-03 | Wisconsin Alumni Research Foundation (Warf) | Vaccines comprising mutant attenuated influenza viruses |
| US12122807B2 (en) | 2019-05-01 | 2024-10-22 | Wisconsin Alumni Research Foundation (Warf) | Influenza virus replication for vaccine development |
| US12144857B2 (en) | 2018-08-20 | 2024-11-19 | Wisconsin Alumni Research Foundation (Warf) | Vectors for eliciting immune responses to non-dominant epitopes in the hemagglutinin (HA) protein |
| US12251436B2 (en) | 2017-10-25 | 2025-03-18 | Wisconsin Alumni Research Foundation (Warf) | Recombinant influenza viruses with stabilized HA for replication in eggs |
| US12290562B2 (en) | 2020-03-25 | 2025-05-06 | Wisconsin Alumni Research Foundation (Warf) | Recombinant multivalent influenza viruses |
| US12343390B2 (en) | 2018-08-07 | 2025-07-01 | Wisconsin Alumni Research Foundation (Warf) | Recombinant biologically contained filovirus vaccine |
| US12364748B2 (en) | 2016-02-19 | 2025-07-22 | Wisconsin Alumni Research Foundation (Warf) | Influenza B virus replication for vaccine development |
| US12410409B2 (en) | 2011-08-26 | 2025-09-09 | Wisconsin Alumni Research Foundation (Warf) | Influenza viruses with mutant PB2 gene segment as live attenuated vaccines |
Families Citing this family (13)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| ES2217967B1 (en) * | 2003-03-31 | 2006-01-01 | Consejo Sup. Investig. Cientificas | PROCEDURE FOR THE PRODUCTION OF EMPTY VIRAL PARTICLES (VLPS) OF THE INFECTIOUS BURSITIS INDUCTOR VIRUS (IBDV), COMPOSITIONS NEEDED FOR ITS POSITIONING AND ITS USE IN THE DEVELOPMENT OF VACCINES AGAINST IBDV. |
| ES2307346B1 (en) * | 2004-01-21 | 2009-11-13 | Consejo Sup. Investig. Cientificas | EMPTY CAPSIDES (VLPS (-VP4)) OF THE VIRUS CAUSING THE INFECTIOUS BURSITIS DISEASE (IBDV), ITS PROCESSING PROCEDURE AND APPLICATIONS. |
| ES2307345B1 (en) * | 2004-01-21 | 2009-11-13 | Consejo Sup. Investig. Cientificas | CHEMICAL EMPTY CAPSIDES OF THE VIRUS CAUSING THE INFECTIOUS BURSITIS DISEASE (IBDV), ITS PROCEDURE FOR OBTAINING AND APPLICATIONS. |
| ES2310062B1 (en) * | 2005-07-15 | 2009-11-13 | Bionostra, S.L. | PSEUDOVIRAL PARTICLES CHEMICAL EMPTY DERIVED FROM VIRUS CAUSING INFECTIOUS BURSITIS DISEASE (IBDV), PROCEDURE OF OBTAINING AND APPLICATIONS. |
| ES2555544T3 (en) | 2006-03-07 | 2016-01-04 | Vaxinnate Corporation | Compositions that include hemagglutinin, preparation methods and methods of use thereof |
| RU2009105099A (en) | 2006-07-14 | 2010-08-27 | Санофи Пастер Байолоджикс Ко. (Us) | CONSTRUCTION OF RECOMBINANT VIRAL VACCINES BY DIRECT TRANSPOSION-MEDIATED INSERATION OF ALIEN IMMUNOLOGICAL DETERMINANTS IN VECTOR VIRUS PROTEINS |
| KR20090096414A (en) | 2006-09-29 | 2009-09-10 | 사노피 파스테르 바이오로직스 씨오 | Recombinant rhino virus vectors |
| AU2009236585B2 (en) | 2008-04-18 | 2013-03-07 | Vaxinnate Corporation | Deletion mutants of flagellin and methods of use |
| AU2013295647B2 (en) | 2012-07-26 | 2018-02-08 | The Henry M. Jackson Foundation For The Advancement Of Military Medicine, Inc. | Multimeric fusion protein vaccine and immunotherapeutic |
| US8932598B2 (en) | 2012-08-28 | 2015-01-13 | Vaxinnate Corporation | Fusion proteins and methods of use |
| HK1208355A1 (en) * | 2012-11-05 | 2016-03-04 | Georgia State University Research Foundation, Inc. | Universal influenza vaccine based on heterologous multiple m2e proteins |
| EP3512874A2 (en) | 2017-11-30 | 2019-07-24 | Grifols Diagnostic Solutions Inc. | Immunoassays and engineered proteins for monitoring antibody treatments to the immune checkpoint inhibitors pd1 and pd-l1 |
| EP4277918A4 (en) * | 2021-01-13 | 2025-07-30 | Purdue Research Foundation | SUPRAMOLECULAR ARRANGEMENTS, COMPOSITIONS AND METHODS FOR THE PREPARATION AND USE THEREOF |
Family Cites Families (9)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| US5041385A (en) * | 1986-11-01 | 1991-08-20 | Oxford Gene Systems Limited | Vector expressing fusion proteins and particles |
| ATE240394T1 (en) | 1992-10-23 | 2003-05-15 | Immunex Corp | METHODS FOR PRODUCING SOLUBLE OLIGOMERIC PROTEINS |
| US5721340A (en) * | 1994-11-28 | 1998-02-24 | The Wistar Institute Of Anatomy & Biology | p53 proteins with altered tetramerization domains |
| WO1999062953A1 (en) * | 1998-06-04 | 1999-12-09 | Shanghai Second Medical University | A human leucine zipper protein gene (bmh) (cblayd06) |
| PL192016B1 (en) * | 1998-11-30 | 2006-08-31 | Cytos Biotechnology Ag | Ordered molecular presentation of antigens, method of preparation and use |
| AU4770300A (en) * | 1999-05-14 | 2000-12-05 | Medical Research Council | Protein scaffold and its use to multimerise monomeric polypeptides |
| IL147270A0 (en) | 1999-07-02 | 2002-08-14 | Genentech Inc | Fusion peptides comprising a peptide ligand domain and a multimerization domain |
| DE19963859A1 (en) * | 1999-12-30 | 2001-07-12 | Apotech Res & Dev Ltd | Bi- or oligomer of a di-, tri-, quattro- or pentamer of recombinant fusion proteins |
| US20020015951A1 (en) | 2000-01-06 | 2002-02-07 | Bader Joel S. | Method of analyzing a nucleic acid |
-
2002
- 2002-01-18 US US10/466,655 patent/US7449188B2/en not_active Expired - Lifetime
- 2002-01-18 WO PCT/EP2002/000628 patent/WO2002074795A2/en not_active Ceased
- 2002-01-18 DK DK02722030T patent/DK1362109T3/en active
- 2002-01-18 CA CA2435000A patent/CA2435000C/en not_active Expired - Lifetime
- 2002-01-18 AT AT02722030T patent/ATE433491T1/en active
- 2002-01-18 ES ES02722030T patent/ES2327719T3/en not_active Expired - Lifetime
- 2002-01-18 EP EP02722030A patent/EP1362109B1/en not_active Expired - Lifetime
- 2002-01-18 AU AU2002252978A patent/AU2002252978B9/en not_active Expired
- 2002-01-18 DE DE60232577T patent/DE60232577D1/en not_active Expired - Lifetime
Cited By (47)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| US8734778B2 (en) | 2002-12-16 | 2014-05-27 | Globeimmune, Inc. | Yeast-based vaccines as immunotherapy |
| US9452210B2 (en) | 2007-07-13 | 2016-09-27 | Medicago Inc. | Influenza virus-like particles (VLPS) comprising hemagglutinin produced within a plant |
| US9458470B2 (en) | 2007-11-27 | 2016-10-04 | Medicago Inc. | Recombinant influenza virus-like particles (VLPs) produced in transgenic plants expressing hemagglutinin |
| US11434497B2 (en) | 2007-11-27 | 2022-09-06 | Medicago Inc. | Recombinant influenza virus-like particles (VLPS) produced in transgenic plants |
| US10190132B2 (en) | 2007-11-27 | 2019-01-29 | Medicago Inc. | Recombinant influenza virus-like particles (VLPs) produced in transgenic plants expressing hemagglutinin |
| WO2009133463A1 (en) * | 2008-04-30 | 2009-11-05 | University Of Copenhagen | Soluble influenza vaccine |
| US8771703B2 (en) | 2008-07-08 | 2014-07-08 | Medicago Inc. | Soluble recombinant influenza antigens |
| WO2010003235A1 (en) * | 2008-07-08 | 2010-01-14 | Medicago Inc. | Soluble recombinant influenza antigens |
| EP2294202A4 (en) * | 2008-07-08 | 2011-10-26 | Medicago Inc | SOLUBLE RECOMBINANT INFLUENZA ANTIGENS |
| AU2009267769B2 (en) * | 2008-07-08 | 2015-07-16 | Medicago Inc. | Soluble recombinant influenza antigens |
| US10272148B2 (en) | 2009-06-24 | 2019-04-30 | Medicago Inc. | Chimeric influenza virus-like particles comprising hemagglutinin |
| US8865182B2 (en) | 2009-07-31 | 2014-10-21 | Paxvax, Inc. | Adenoviral-based vectors |
| US11826419B2 (en) | 2009-09-22 | 2023-11-28 | Medicago Inc. | Method of preparing plant-derived VLPs |
| US11833200B2 (en) | 2009-09-22 | 2023-12-05 | Medicago Inc. | Method of preparing plant-derived proteins |
| US12076387B2 (en) | 2010-03-23 | 2024-09-03 | Wisconsin Alumni Research Foundation (Warf) | Vaccines comprising mutant attenuated influenza viruses |
| WO2011126370A1 (en) * | 2010-04-09 | 2011-10-13 | Universiteit Utrecht Holding B.V. | Recombinant multimeric influenza proteins |
| AU2011280259C1 (en) * | 2010-07-23 | 2018-06-07 | Erasmus University Rotterdam Medical Center | Influenza vaccine |
| KR102143105B1 (en) * | 2010-07-23 | 2020-08-11 | 이스코노바 에이비 | Influenza vaccine |
| CN107281478A (en) * | 2010-07-23 | 2017-10-24 | 诺瓦瓦克斯公司 | Influenza vaccines |
| WO2012011868A1 (en) * | 2010-07-23 | 2012-01-26 | Osterhaus A D M E | Influenza vaccine |
| KR20170141268A (en) * | 2010-07-23 | 2017-12-22 | 이스코노바 에이비 | Influenza vaccine |
| EP3272359A1 (en) * | 2010-07-23 | 2018-01-24 | Novavax AB | Influenza vaccine |
| RU2583297C2 (en) * | 2010-07-23 | 2016-05-10 | Исконова Аб | Influenza vaccine |
| AU2011280259B2 (en) * | 2010-07-23 | 2014-05-22 | Erasmus University Rotterdam Medical Center | Influenza vaccine |
| EP2595653A4 (en) * | 2010-07-23 | 2014-03-12 | Univ Erasmus Medical Ct | INFLUENZA VACCINE |
| US10485863B2 (en) | 2010-07-23 | 2019-11-26 | Novavax AB | Influenza vaccine |
| US10736958B2 (en) | 2010-07-23 | 2020-08-11 | Novavax AB | Influenza vaccine |
| AU2011280259A8 (en) * | 2010-07-23 | 2013-02-28 | Erasmus University Rotterdam Medical Center | Influenza vaccine |
| CN103052401A (en) * | 2010-07-23 | 2013-04-17 | 伊斯克诺瓦公司 | Flu vaccine |
| WO2012128628A1 (en) * | 2011-03-22 | 2012-09-27 | Mucosis B.V. | Immunogenic compositions in particulate form and methods for producing the same |
| US9585953B2 (en) | 2011-03-22 | 2017-03-07 | Mucosis B.V. | Immunogenic compositions in particulate form and methods for producing the same |
| US9815873B2 (en) | 2011-03-23 | 2017-11-14 | Medicago Inc. | Method for recovering plant-derived proteins |
| US12410409B2 (en) | 2011-08-26 | 2025-09-09 | Wisconsin Alumni Research Foundation (Warf) | Influenza viruses with mutant PB2 gene segment as live attenuated vaccines |
| US11802273B2 (en) | 2014-06-20 | 2023-10-31 | Wisconsin Alumni Research Foundation (Warf) | Mutations that confer genetic stability to additional genes in influenza viruses |
| US12364748B2 (en) | 2016-02-19 | 2025-07-22 | Wisconsin Alumni Research Foundation (Warf) | Influenza B virus replication for vaccine development |
| US12251436B2 (en) | 2017-10-25 | 2025-03-18 | Wisconsin Alumni Research Foundation (Warf) | Recombinant influenza viruses with stabilized HA for replication in eggs |
| US12343390B2 (en) | 2018-08-07 | 2025-07-01 | Wisconsin Alumni Research Foundation (Warf) | Recombinant biologically contained filovirus vaccine |
| US12144857B2 (en) | 2018-08-20 | 2024-11-19 | Wisconsin Alumni Research Foundation (Warf) | Vectors for eliciting immune responses to non-dominant epitopes in the hemagglutinin (HA) protein |
| US12258557B2 (en) | 2019-02-08 | 2025-03-25 | Wisconsin Alumni Research Foundation (Warf) | Humanized cell line |
| US11851648B2 (en) | 2019-02-08 | 2023-12-26 | Wisconsin Alumni Research Foundation (Warf) | Humanized cell line |
| US12122807B2 (en) | 2019-05-01 | 2024-10-22 | Wisconsin Alumni Research Foundation (Warf) | Influenza virus replication for vaccine development |
| US11807872B2 (en) | 2019-08-27 | 2023-11-07 | Wisconsin Alumni Research Foundation (Warf) | Recombinant influenza viruses with stabilized HA for replication in eggs |
| US11739303B2 (en) | 2020-01-24 | 2023-08-29 | Wisconsin Alumni Research Foundation (Warf) | Recombinant influenza viruses with stabilized NA |
| JP2023511444A (en) * | 2020-01-24 | 2023-03-17 | ウィスコンシン アルムニ リサーチ ファンデイション | Recombinant influenza virus with stabilized NA |
| US12365880B2 (en) | 2020-01-24 | 2025-07-22 | The University Of Tokyo | Recombinant influenza viruses with stabilized NA |
| WO2021150874A1 (en) * | 2020-01-24 | 2021-07-29 | Wisconsin Alumni Research Foundation (Warf) | Recombinant influenza viruses with stabilized na |
| US12290562B2 (en) | 2020-03-25 | 2025-05-06 | Wisconsin Alumni Research Foundation (Warf) | Recombinant multivalent influenza viruses |
Also Published As
| Publication number | Publication date |
|---|---|
| US20040116664A1 (en) | 2004-06-17 |
| AU2002252978B2 (en) | 2006-12-07 |
| US7449188B2 (en) | 2008-11-11 |
| DE60232577D1 (en) | 2009-07-23 |
| EP1362109B1 (en) | 2009-06-10 |
| CA2435000C (en) | 2014-03-25 |
| ATE433491T1 (en) | 2009-06-15 |
| CA2435000A1 (en) | 2002-09-26 |
| DK1362109T3 (en) | 2009-07-27 |
| EP1362109A2 (en) | 2003-11-19 |
| ES2327719T3 (en) | 2009-11-03 |
| AU2002252978B9 (en) | 2007-02-01 |
| AU2002252978A1 (en) | 2002-10-03 |
| WO2002074795A3 (en) | 2003-09-04 |
Similar Documents
| Publication | Publication Date | Title |
|---|---|---|
| AU2002252978B2 (en) | Oligomeric complexes of chimeric proteins with enhanced immunogenic potential | |
| US11905314B2 (en) | Influenza virus vaccines and uses thereof | |
| CA2913859C (en) | Influenza virus vaccines and uses thereof | |
| CN107074912A (en) | Influenza virus vaccine and application thereof | |
| US20230250135A1 (en) | Influenza virus vaccines and uses thereof | |
| Spitsin et al. | Immunological assessment of plant-derived avian flu H5/HA1 variants | |
| US20240335525A1 (en) | Truncated influenza neuraminidase and methods of using the same | |
| IL294808A (en) | Pyrido[2,3-e]oxazine derivatives as agricultural chemicals | |
| Choi et al. | Immune response induced by the TAT-conjugated influenza M2e in mice | |
| WO2009133463A1 (en) | Soluble influenza vaccine | |
| HK40031633A (en) | Influenza virus vaccines and uses thereof | |
| HK40031633B (en) | Influenza virus vaccines and uses thereof | |
| EA045051B1 (en) | VACCINES AGAINST THE FLU VIRUS AND WAYS OF THEIR APPLICATION | |
| OA19766A (en) | Influenza virus vaccines and uses thereof. | |
| Spitsin et al. | As submitted to: Vaccine and later published as:“Immunological assessment of plant-derived avian flu H5/HA1 variants.” In Vaccine. Volume 27, Issue 9, 25 February 2009, Pages 1289-1292 | |
| Conrad et al. | A Plant-Based Artificial Haemagglutinin (A/H5N1) Strongly Induced Neutralizing Immune Responses in Mice |
Legal Events
| Date | Code | Title | Description |
|---|---|---|---|
| AK | Designated states |
Kind code of ref document: A2 Designated state(s): AE AG AL AM AT AU AZ BA BB BG BR BY BZ CA CH CN CO CR CU CZ DE DK DM DZ EC EE ES FI GB GD GE GH GM HR HU ID IL IN IS JP KE KG KP KR KZ LC LK LR LS LT LU LV MA MD MG MK MN MW MX MZ NO NZ OM PH PL PT RO RU SD SE SG SI SK SL TJ TM TN TR TT TZ UA UG US UZ VN YU ZA ZM ZW |
|
| AL | Designated countries for regional patents |
Kind code of ref document: A2 Designated state(s): GH GM KE LS MW MZ SD SL SZ TZ UG ZM ZW AM AZ BY KG KZ MD RU TJ TM AT BE CH CY DE DK ES FI FR GB GR IE IT LU MC NL PT SE TR BF BJ CF CG CI CM GA GN GQ GW ML MR NE SN TD TG |
|
| DFPE | Request for preliminary examination filed prior to expiration of 19th month from priority date (pct application filed before 20040101) | ||
| 121 | Ep: the epo has been informed by wipo that ep was designated in this application | ||
| WWE | Wipo information: entry into national phase |
Ref document number: 2002252978 Country of ref document: AU |
|
| WWE | Wipo information: entry into national phase |
Ref document number: 2002722030 Country of ref document: EP |
|
| WWE | Wipo information: entry into national phase |
Ref document number: 2435000 Country of ref document: CA |
|
| WWE | Wipo information: entry into national phase |
Ref document number: 10466655 Country of ref document: US |
|
| WWP | Wipo information: published in national office |
Ref document number: 2002722030 Country of ref document: EP |
|
| REG | Reference to national code |
Ref country code: DE Ref legal event code: 8642 |
|
| NENP | Non-entry into the national phase |
Ref country code: JP |
|
| WWW | Wipo information: withdrawn in national office |
Country of ref document: JP |