WO2007073845A2 - Polypeptide having esterase activity and recombinant esterase and use thereof - Google Patents
Polypeptide having esterase activity and recombinant esterase and use thereof Download PDFInfo
- Publication number
- WO2007073845A2 WO2007073845A2 PCT/EP2006/011832 EP2006011832W WO2007073845A2 WO 2007073845 A2 WO2007073845 A2 WO 2007073845A2 EP 2006011832 W EP2006011832 W EP 2006011832W WO 2007073845 A2 WO2007073845 A2 WO 2007073845A2
- Authority
- WO
- WIPO (PCT)
- Prior art keywords
- alkyl
- esterase
- halopent
- polypeptide
- formula
- Prior art date
- Legal status (The legal status is an assumption and is not a legal conclusion. Google has not performed a legal analysis and makes no representation as to the accuracy of the status listed.)
- Ceased
Links
Classifications
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N9/00—Enzymes; Proenzymes; Compositions thereof; Processes for preparing, activating, inhibiting, separating or purifying enzymes
- C12N9/14—Hydrolases (3)
- C12N9/16—Hydrolases (3) acting on ester bonds (3.1)
- C12N9/18—Carboxylic ester hydrolases (3.1.1)
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N15/00—Mutation or genetic engineering; DNA or RNA concerning genetic engineering, vectors, e.g. plasmids, or their isolation, preparation or purification; Use of hosts therefor
- C12N15/09—Recombinant DNA-technology
- C12N15/11—DNA or RNA fragments; Modified forms thereof; Non-coding nucleic acids having a biological activity
- C12N15/52—Genes encoding for enzymes or proenzymes
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12P—FERMENTATION OR ENZYME-USING PROCESSES TO SYNTHESISE A DESIRED CHEMICAL COMPOUND OR COMPOSITION OR TO SEPARATE OPTICAL ISOMERS FROM A RACEMIC MIXTURE
- C12P41/00—Processes using enzymes or microorganisms to separate optical isomers from a racemic mixture
- C12P41/003—Processes using enzymes or microorganisms to separate optical isomers from a racemic mixture by ester formation, lactone formation or the inverse reactions
- C12P41/005—Processes using enzymes or microorganisms to separate optical isomers from a racemic mixture by ester formation, lactone formation or the inverse reactions by esterification of carboxylic acid groups in the enantiomers or the inverse reaction
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12P—FERMENTATION OR ENZYME-USING PROCESSES TO SYNTHESISE A DESIRED CHEMICAL COMPOUND OR COMPOSITION OR TO SEPARATE OPTICAL ISOMERS FROM A RACEMIC MIXTURE
- C12P7/00—Preparation of oxygen-containing organic compounds
- C12P7/02—Preparation of oxygen-containing organic compounds containing a hydroxy group
Definitions
- Novel polypeptide having esterase activity and recombinant esterase and use thereof
- the invention relates to a novel polypeptide having esterase activity, especially having 2-alkyl-5- halopent-4-enecarboxylesterase activity, and to an enzymatically active recombinant protein having esterase activity and to the use thereof for resolving racemates of 2-alkyl-5-halopent-4-enecarboxylic ester enantiomer mixtures.
- Enantiomerically enriched 2-alkyl-5-halopent-4- enecarboxylic acids and their esters are valuable intermediates for preparing pharmaceuticals, such as, for instance, for delta-amino-gamma-hydroxy-omega- arylalkanecarboxamides, which have renin-inhibiting properties and can be used as antihypertensive agents in pharmaceutical preparations.
- Esterases are generally employed in the resolution of racemates and asymmetrization.
- esterase extracts from pig liver is known on the preparative scale.
- Pig liver esterase (PLE) was isolated long ago from natural sources, and its activity has also been known for a long time (Simonds, J. P. (1919) Amer. J. Physiol. 48, 141; Bamann, E. et al . (1934) Hoppe-Seyler Z. 229, 15; Falconer J. S. and Taylor, D. B. (1946) Biochem. J. 40, 831-834) .
- racemic 2-alkyl-5-halopent-4- enecarboxylic esters is not described in any of these articles.
- rAPLE whose amino acid sequence differs in 21 of a total of 548 amino acids from the known PLE sequence.
- the novel rAPLE differs in the amino acid sequence also from the known pig intestinal carboxylesterase (PICE) in 12 of a total of 548 amino acids.
- PICE pig intestinal carboxylesterase
- the present invention accordingly relates to a polypeptide having esterase activity, which comprises the amino acid sequence SEQ. ID. No. 1.
- the present invention further relates to a novel recombinant protein having esterase activity, which comprises the amino acid sequence SEQ. ID. No. 1.
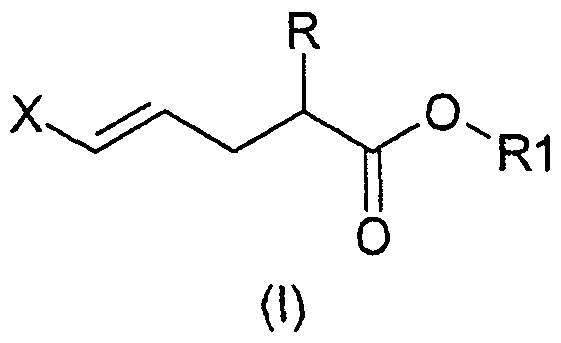
- the polypeptide and the recombinant rAPLE of the invention have the ability to resolve stereoselectively racemic 2-alkyl-5-halopent-4-enecarboxylic esters of the formula (I) in which R is a d-C 6 -alkyl radical, Ri is d-C 4 -alkyl and X is chlorine, bromine or iodine.
- the polypeptide of the invention having esterase activity, and the novel recombinant esterase rAPLE differ, as stated above, in 21 of a total of 548 amino acids of the known sequence disclosed in FEBS Lett. (1991), 293, 37-41 and in 12 of a total of 548 amino acids from the known PICE protein disclosed in David et al., (1998) Eur. J. Biochem. 257, 142-148.
- sequence of the protein of the novel rAPLE of the invention differs in the following amino acid positions from the known sequence of the PLE protein:
- the protein of the invention and the novel recombinant rAPLE may moreover be in the form of a modified sequence as shown in SEQ ID No 1, which can be obtained for example by usual modifications such as, for instance, exchange, deletion or attachment of amino acid(s) in the sequence at the N or C terminus, such as, for instance, GluAlaGluAla from the ⁇ factor signal sequence, or by fusion to other proteins.
- the invention also further includes muteins having modifications within the protein sequence of the enzyme of the invention having the appropriate activity, in particular on 2-alkyl-5-halopent-4-enecarboxylic esters.
- Muteins can be obtained for example by modifications of the DNA which codes for the enzyme of the invention, by known mutagenesis techniques (random mutagenesis, site-directed mutagenesis, directed evolution, gene shuffling etc.) so that the DNA codes for an enzyme which differs at least by one amino acid from the enzyme of the invention, and subsequent expression of the modified DNA in a suitable host cell.
- the invention thus also includes modified DNA sequences as shown in SEQ ID. No 1, obtained by the mutations, deletions, extensions, fusions described above, and which code for enzymes having the desired esterase activity.
- Esterase activity is defined in this connection as the ability to resolve racemates of 2-alkyl-5-halopent-4-enecarboxylic esters of the formula (I) .
- the polypeptide of the invention and the recombinant rAPLE can be prepared as described below:
- mRNA is isolated from pig liver using a suitable kit, and then the cDNA is generated by reverse transcription based on the mRNA extract. Subsequently, specific PCR primers based on the sequence of the known pig liver esterase gene of GenBank accesssion No. X63323 (Matsushima et al . , 1991) is prepared, followed by amplification and cloning. These specific primers are:
- Primer 1 5 ' -CAGAATTCATGGCTATCGGGCAGCCAGCCTCGC-S '
- Primer 2 5 ' -CCGGAATTCAGCCTCCCCTTCACAGCTCAG-B '
- This part of the primers which comprises the appropriate nucleotide sequences coding for the PLE protein and which is obligatorily present in the primers is in bold script.
- the other sequence part of the primers comprises for example information for cleavage sites for restriction endonucleases (in italics) or sequence elements which are important for expression. This part may vary in the preparation of the rAPLE of the invention.
- Amplification then takes place with primers 1 and 2 by prior art PCR methods .
- the PCR product is subsequently used to prepare by prior art methods expression constructs for heterologous expression of the encoded rAPLE protein in suitable host organisms. This preferably entails the PCR product being initially cloned into suitable plasmid vectors.
- the recombinant plasmids obtained in this way are then transformed into a suitable host, for example
- the present invention further relates to a nucleic acid or nucleotide sequence which codes for the polypeptide of the invention and the recombinant esterase rAPLE.
- such a nucleic acid has the nucleotide sequence shown in SEQ. ID. No. 2.
- the invention also relates further to nucleotide sequences which include a nucleotide sequence which codes for the polypeptide of the invention and the recombinant esterase rAPLE, or comprises the nucleotide sequence shown in SEQ. ID. No. 2.
- a further possibility is to prepare appropriate oligonucleotides corresponding to nucleic acid sequences according to the present invention which code for the esterase of the invention by standardized synthetic techniques, for example with use of automated DNA synthesizers.
- the purely synthetic preparation of the nucleic acid sequences which code for the esterase of the invention is particularly advantageous for use in the production of pharmaceuticals or their intermediates, because enzymes are thus not obtained from animal sources .
- the known pig liver esterase (PLE, Swiss-Prot ID Q29550) comprises an N-terminal signal sequence and a C-terminal ER retention signal, the last 4 amino acids HAEL.
- Suitable host cells in this connection are for example microorganisms, animal cell lines and plants. Both prokaryotic and eukaryotic microorganisms can be employed. Preferred prokarytic hosts (bacteria) are
- B.amyloliguefaciens B.amyloliguefaciens
- Pseudomonas e.g. P. fluorescens, P.putida
- Streptomyces e.g. S.lividans, S.tendae
- Eukaryotic microorganisms are preferred, and fungi are particularly preferred. Examples thereof are Saccharomyces cerevisiae, Pichia pastoris, Kluyveromyces lactis or Aspergillus sp.. Expression may be secretory or intracellular and both inducible and constitutive.
- the proteins are preferably expressed in a secretory manner, in which case vectors in which the sequences of PLE and APLE are linked N-terminally to the ⁇ factor signal sequence of S. cerevisiae are preferably constructed.
- a further preferred expression is inducible expression of constructs with or without ER retention signal.
- constructs having the ER retention signal can also be expressed and lead to an rAPLE which is capable of selective resolution of racemic 2-alkyl-5- halopent-4-enecarboxylic esters.
- amino acid sequence of the novel esterase rAPLE which is derived from the nucleotide sequence of the APLE gene is depicted in SEQ ID No. 1.
- novel polypeptide or the rAPLE protein is able, in contrast to the known rPLE, in each case obtained by expression of the DNA segments coding for APLE and PLE, respectively, for example in P. pastoris cells, to resolve racemic 2-alkyl-5-halopent-4-enecarboxylic esters stereoselectively .
- the invention accordingly further relates to the use of the polypeptide having esterase activity and of the recombinant esterase (rAPLE) of the invention, which have at least 80% identity to the sequence shown in SEQ ID No. 1, for resolving racemates of 2-alkyl-5- halopent-4-enecarboxylic esters of the formula (I)
- R is a Ci-Ce-alkyl radical
- Ri is d-C 4 -alkyl
- X is chlorine, bromine or iodine.
- polypeptide having esterase activity and the recombinant esterase (rAPLE) of the invention preferably have at least 90%, particularly preferably at least 98%, identity to the sequence of the protein shown in SEQ ID No. 1. It is also possible to employ polypeptide having an esterase activity or the recombinant esterase (rAPLE) of the invention with modified DNA sequences shown in SEQ ID. No. 1, obtained by usual modifications such as, for instance, mutations, deletions, extensions, fusions, which code for enzymes having the desired esterase activity.
- R is a C 1 -C 6 -alky1 radical
- A is equal to H
- R 1 where R 1 may be Ci-C 4 -alkyl, or R 2 , where R 2 is an alkyl group, but is not equal to R 1
- X is chlorine, bromine or iodine, are obtained by an enantiomeric mixture of a 2-alkyl-5-halopent-4-enecarboxylic ester of the formula (I)
- R, R 1 and X are as defined above, being converted by means of the polypeptide of the invention or of the rAPLE of the invention in the presence of water or an alcohol of the formula R 2 OH, where R 2 is an alkyl group which is not equal to R 1 , as nucleophile, and a) either the remaining enantiomerically enriched 2-alkyl-5-halopent-4-enecarboxylic ester of the formula (II) with A equal to R 1 being isolated or b) if an alcohol is employed as nucleophile, the resulting enantiomerically enriched 2-alkyl-5- halopent-4-enecarboxylic ester of the formula (II) with A equal to R 2 being isolated, or c) if water is employed as nucleophile, the resulting 2-alkyl-5-halopent-4-enecarboxylic acid of the formula (II) with A equal to H being isolated.
- R in the formula (II) is a Ci-C 6 -alkyl radical such as, for instance, methyl, ethyl, n- and i-propyl, n- , i- and t-butyl, pentyl and hexyl .
- Ci-C 4 -Alkyl radicals are preferred, and the i-propyl radical is particularly preferred.
- A is H, Ri, where R 1 is a Ci-C 4 -alkyl radical, preferably a Ci-C 2 -alkyl radical and particularly preferably a methyl radical, or R 2 , where R 2 is an alkyl radical which is not equal to Ri. R 2 is particularly preferably a Ci-C 3 -alkyl radical.
- X is chlorine, bromine or iodine, preferably chlorine.
- Enantiomerically enriched compounds mean in this connection those which exhibit an enantiomeric excess
- the enzyme of the invention can moreover be used in any form.
- dispersion as solution, immobilized, as crude enzyme, as enzyme which has been obtained from its source by a combination of known purification methods, as whole cells (where appropriate immobilized and/or permeabilized) which have the required enzymatic activity (naturally or through genetic modifications) or in a lysate of such cells.
- the reaction temperature for the conversion of the invention is normally between 0 and 9O 0 C, preferably between 10 and 6O 0 C.
- the pH of the reaction solution is between 4 and 11, preferably between 6 and 9.
- solvents which can be employed are water, a mixture of water with a water-miscible solvent, for example with an alcohol such as, for instance, methanol, ethanol, isopropanol, t-butanol, etc., dioxane, tetrahydrofuran, acetone or dimethyl sulfoxide or a two-phase system of water and of a water- immiscible solvent, for example an aromatic compound such as, for instance, toluene, xylene, etc., an alkane such as, for instance, hexane, heptane, cyclohexane, etc., ether such as, for instance, diisopropyl ether, methyl t-butyl ether, etc.
- an alcohol such as, for instance, methanol, ethanol, isopropanol, t-butanol, etc.
- dioxane tetrahydrofuran
- the solvent preferably employed is the alcohol R 2 OH where R 2 is an alkyl group which is not, however, equal to Ri.
- R 2 is an alkyl group which is not, however, equal to Ri.
- an organic solvent such as, for instance, tetrahydrofuran, heptane, toluene, hexane, CH 3 CN, methyl t-butyl ether etc.
- the desired final product is isolated.
- This may be either the remaining enantiomerically enriched 2-alkyl-5-halopent-4-enecarboxylic ester of the formula (II) with A equal to Ri, or if water is the nucleophile the enantiomerically enriched 2-alkyl-5- halopent-4-enecarboxylic acid of the formula (II) with A equal to H which has formed, or if the alcohol is the nucleophile the enantiomerically enriched 2-alkyl-5- halopent-4-enecarboxylic ester of the formula (II) with A equal to R 2 .
- the isolation can take place for example by conventional methods such as, for instance, extraction, crystallization, column chromatography, distillation, etc.
- the method of the invention results in the corresponding acids or esters of the formula (I) in theoretical yields of up to 98% yield and with an e.e. of up to >99%.
- Example 1 mRNA isolation and generation of cDNA
- Example 2 Amplification and cloning of cDNA fragments from pig liver
- Primer 1 5 1 -CAGM7TCATGGCTATCGGGCAGCCAGCCTCGC-3 1 (SEQ ID. No.3)
- Primer 2 5'-CCGGyAA7TCAGCCTCCCCTTCACAGCTCAG -3' (SEQ ID No.4)
- This PCR resulted in a DNA fragment with a size of 1.8 kb (found by agarose gel electrophoresis) .
- This PCR product was then purified using the Qiaquick kit (Qiagen, Hilden, Germany) in accordance with the manual included.
- the vectors were then transformed into TOPlO electrocompetent cells prepared in accordance with 'Current Protocols in Molecular Biology' .
- Example 3 Introduction of the ⁇ factor signal sequence and variations of the C-terminal end.
- vectors in which the sequence of PLE and APLE was connected N-terminally to the ⁇ factor start sequence of the cloning vector pPICZ ⁇ were constructed.
- constructs in which the C-terminal tetrapeptide HAEL was deleted were prepared.
- PCR I The EcoRIalphal/alphaPLE2 primer pair was used to amplify the ⁇ factor signal sequence of the cloning vector pPICZ ⁇ (Invitrogen) .
- the PCR was carried out in a 50 ⁇ l mixture (2 ng of template, 0.5 ⁇ M of each primer, 0.2 mM dNTPs, 1 U of the- Phusion DNA polymerase (Finnzymes) all in lxPhusion HF buffer in accordance with the * Phusion High-Fidelity DNA Polymerase' manual (Finnzymes) ) . Denaturation at 95 0 C for 3 minutes was followed by amplification in 30 cycles (30 sec 95 0 C, 30 sec 57°C, 15 sec 72 0 C) and a final step at 72 0 C for 7 min.
- PCR II The PLE and APLE sequences were amplified from pHILZ plasmids using either the PLEalphal/EcoRIPLE+ER2 primer pair or the PLEalphal/EcoRIPLE2 (deletion of the C-terminal HAEL tetrapeptide) primer pair. These PCRs were again carried out in 50 ⁇ l mixtures (2 ng of template, 0.5 ⁇ M of each primer, 0.2 mM dNTPs, 1 U of the Phusion DNA polymerase (Finnzymes) all in lxPhusion HF buffer in accordance with the 'Phusion High-Fidelity DNA Polymerase' Manual (Finnzymes) ) . A denaturation at 95 0 C for 3 minutes was followed by amplification in 30 cycles (30 sec 95 0 C, 30 sec 57 0 C, 15 sec 72 0 C) and a final step at 72 0 C for 7 min.
- PCR III 3 ⁇ l of the products from PCR 1 and PCR II were used to combine these two products by primerless PCR.
- the extension was carried out in a 45 ⁇ l mixture with 0.2 mM dNTPs, I U of the Phusion DNA polymerase (Finnzymes) all in lxPhusion HF buffer.
- the reaction mixture was heated at 95 0 C for 3 minutes and then 10 cycles with 30 sec at 95 0 C and 45 sec at 72 0 C were carried out.
- 5 ⁇ l of primer mix (3 ⁇ l of water, 1 ⁇ l of 5 ⁇ M EcoRIalphal primer and 1 ⁇ l of 5 ⁇ M EcoRIPLE+ER2 or EcoRIPLE2 primer) were added.
- alphaPLE2 5'-GAGGCTGGCTGCCCAGCTTCAGCCTCTCTTTTCTCG-3' (SEQ ID No. 6)
- PLEalphal 5 1 -AGAGAGGCTGAAGCTGGGCAGCCAGCCTCGCCG-3 1 (SEQ ID No. 7)
- ECORIPLE+ER2 5'-ATGG ⁇ CCG/A/ ⁇ 7TCTCACAGCTCAGCATGCTTTATCTTG-3' (SEQ ID No. 8)
- Example 4 Construction of expression constructs for the heterologous expression of pig liver esterases in Pichia pastoris
- the overlapping extension PCR products from example 3 were purified using the Qiaquick kit (Qiagen, Hilden, Germany) in accordance with the manual included. About 0.1 ⁇ g of the purified PCR products was cut using the EcoRI restriction endonuclease and cloned via the EcoRI cleavage site into the plasmid vector pGAPZ A (Invitrogen) .
- Example 5 Constitutive expression of pig liver esterases in Pichia pastoris
- the plasmids pGAPZ A PLE-ER, pGAPZ A PLE+ER, pGAPZ A APLE-ER and pGAPZ A APLE+ER were transformed into P. pastoris X-33.
- the transformation took place in accordance with the instructions of the protocol for the Pichia Expressions kit from Invitrogen.
- the transformants were selected on YPD plates (1% yeast extract, 2% peptone, 2% D-glucose, 2% agar) which contained 100 mg/1 zeocin.
- 52 zeocin-resistant clones were streaked onto YPD plates with 100 mg/1 zeocin and preserved in 15% glycerol.
- P. pastoris transformants were cultured on YPD plates with 100 mg/1 zeocin at 3O 0 C for 48 h. The cells were lifted onto Whatman 541 hardened ashless 70 mm0 filters and air-dried. The filters were incubated with a solution of 6 mg of ⁇ -naphthyl acetate (Sigma, dissolved in 500 ⁇ l of acetone), 2.5 mg of tetrazotized o-dianisidine (Fast Blue Salt BN, Sigma, dissolved in 125 ⁇ l of water) and 5 ml of 0.1 M potassium phosphate buffer, pH 7, in order to visualize the esterase activity by a color reaction.
- ⁇ -naphthyl acetate Sigma, dissolved in 500 ⁇ l of acetone
- tetrazotized o-dianisidine Fest Blue Salt BN, Sigma, dissolved in 125 ⁇ l of water
- P. pastoris transformants as described in example 6 were cultured on YPD plates with 100 mg/1 zeocin at 30 0 C for 48 h. The cells were lifted onto Whatman 541 hardened ashless 70 mm0 filters and air-dried. The filters were incubated either with substrate solution A (100 ⁇ l of racemic methyl 5-chloro-2- (1-methylethyl) -4- pentenoate, 200 ⁇ l of 0.1 M potassium phosphate buffer, pH 8; 150 ⁇ l of 10 mg/ml phenol red; 450 ⁇ l of DMSO; 650 ⁇ l of H 2 O) or with substrate solution B (identical to solution A but employing methyl (2S, 4E) -5-chloro-2- (1-methylethyl) -4 -pentenoate instead of the racemate) . Owing to the specific esterase activity on the substrates, the liberation of acid on hydrolysis of the ester substrate results in a pH decrease which in turn leads to a change in the color
- Transformants obtained with the plasmids pGAPZ A PLE-ER or pGAPZ A PLE+ER showed no reaction with substrate solutions A or B under the same conditions. This showed that the recombinant rAPLE has a substrate specificity different from recombinant rPLE and that hydrolysis of methyl 5-chloro-2- (1-methylethyl) -4- pentenoate using rAPLE takes place stereoselectively for the (R) enantiomer.
- pastoris cultures (72 h at 100 rpm and 28 0 C in 250 ml of YPD medium in 2 1 Erlenmeyer flasks with baffles) which contained either the plasmid pGAPZ A APLE-ER or an empty pGAPZ A plasmid (control strain) .
- the proteins were separated on a 12.5% polyacrylamide gel (4% stacking gel) and stained with Coomassie Brilliant Blue R250 for detection.
- the SDS- PAGE shows a protein band with the expected size for rAPLE (-60 kDa) in the yeast strain having the pGAPZ A APLE plasmid, but not in the control strain (figure 2) .
- the commercially available pig liver esterase which was also analyzed for comparison showed two protein bands in the same size range (arrow in figure 2) .
- Example 9 Induced expression of pig liver esterases with the AOXl promoter
- the plasmids pGAPZ A PLE-ER, pGAPZ A PLE+ER, pGAPZ A APLE-ER and pGAPZ A APLE+ER were cut with the restriction endonuclease Xhol, and the respective fragments coding for APLE and PLE proteins, with or without ER retention signal, were cloned via the Xhol cleavage site into the pPIC9 vector (Invitrogen) . Correct orientation of the fragments in relation to the AOXl promoter was checked by means of control cuts with the restriction endonuclease Ncol .
- the vectors having the AOXl promoter were named, in analogy to the plasmids named in example 4, pPIC9 PLE-ER, pPIC9 PLE+ER, pPIC9 APLE-ER and pPIC9 APLE+ER, linearized with Sail and transformed into P. pastoris KM71. Transformation and selection for His prototrophy took place in accordance with the instructions of the Pichia expression kit from Invitrogen. Selected transformants and the KM71 strain were cultured on complete medium in accordance with the Pichia expression kit from Invitrogen overnight and induced with 1% methanol for 48 h.
Landscapes
- Chemical & Material Sciences (AREA)
- Organic Chemistry (AREA)
- Life Sciences & Earth Sciences (AREA)
- Engineering & Computer Science (AREA)
- Wood Science & Technology (AREA)
- Zoology (AREA)
- Health & Medical Sciences (AREA)
- Genetics & Genomics (AREA)
- Bioinformatics & Cheminformatics (AREA)
- Biotechnology (AREA)
- General Engineering & Computer Science (AREA)
- Microbiology (AREA)
- Biochemistry (AREA)
- General Health & Medical Sciences (AREA)
- General Chemical & Material Sciences (AREA)
- Chemical Kinetics & Catalysis (AREA)
- Biomedical Technology (AREA)
- Molecular Biology (AREA)
- Medicinal Chemistry (AREA)
- Analytical Chemistry (AREA)
- Physics & Mathematics (AREA)
- Biophysics (AREA)
- Plant Pathology (AREA)
- Enzymes And Modification Thereof (AREA)
- Micro-Organisms Or Cultivation Processes Thereof (AREA)
- Preparation Of Compounds By Using Micro-Organisms (AREA)
Abstract
Description



Claims


Priority Applications (14)
| Application Number | Priority Date | Filing Date | Title |
|---|---|---|---|
| CN200680049665.5A CN101351548B (en) | 2005-12-27 | 2006-12-08 | There is the polypeptide of esterase activity and the esterase of restructuring and uses thereof |
| CA2635380A CA2635380C (en) | 2005-12-27 | 2006-12-08 | Polypeptide having esterase activity and recombinant esterase and use thereof |
| PL06829433T PL1966373T3 (en) | 2005-12-27 | 2006-12-08 | Polypeptide having esterase activity and recombinant esterase and use thereof |
| KR1020087018341A KR101388391B1 (en) | 2005-12-27 | 2006-12-08 | Polypeptide having esterase activity and recombinant esterase and use thereof |
| AT06829433T ATE549400T1 (en) | 2005-12-27 | 2006-12-08 | POLYPEPTIDE WITH ESTERASE ACTIVITY AND RECOMBINANT ESTERASE AND USE THEREOF |
| US12/159,547 US8158393B2 (en) | 2005-12-27 | 2006-12-08 | Polypeptide having esterase activity and recombinant esterase and use thereof |
| ES06829433T ES2383702T3 (en) | 2005-12-27 | 2006-12-08 | New polypeptide that has an activity of esterase, and recombinant esterase and its use |
| BRPI0621280A BRPI0621280A8 (en) | 2005-12-27 | 2006-12-08 | POLYPEPTIDES HAVING ESTERASE AND RECOMBINANT ESTERASE ACTIVITIES AND THEIR USES |
| EP06829433A EP1966373B1 (en) | 2005-12-27 | 2006-12-08 | Polypeptide having esterase activity and recombinant esterase and use thereof |
| JP2008547868A JP5119166B2 (en) | 2005-12-27 | 2006-12-08 | Novel polypeptides having esterase activity and recombinant esterases and their use |
| HK09106051.4A HK1128306B (en) | 2005-12-27 | 2006-12-08 | Polypeptide having esterase activity and ecombinant esterase and use thereof |
| IL192400A IL192400A (en) | 2005-12-27 | 2008-06-23 | Polypeptide having esterase activity and recombinant esterase and use thereof |
| NO20082864A NO343225B1 (en) | 2005-12-27 | 2008-06-27 | New polypeptide with esterase activity and recombinant esterase and its use |
| US13/417,734 US8642312B2 (en) | 2005-12-27 | 2012-03-12 | Polypeptide having esterase activity and recombinant esterase and use thereof |
Applications Claiming Priority (2)
| Application Number | Priority Date | Filing Date | Title |
|---|---|---|---|
| AT0208105A AT502990A1 (en) | 2005-12-27 | 2005-12-27 | NEW POLYPEPTIDE WITH ESTERASE ACTIVITY, AND RECOMBINANT ESTERASE AND THEIR USE |
| ATA2081/2005 | 2005-12-27 |
Related Child Applications (2)
| Application Number | Title | Priority Date | Filing Date |
|---|---|---|---|
| US12/159,547 A-371-Of-International US8158393B2 (en) | 2005-12-27 | 2006-12-08 | Polypeptide having esterase activity and recombinant esterase and use thereof |
| US13/417,734 Division US8642312B2 (en) | 2005-12-27 | 2012-03-12 | Polypeptide having esterase activity and recombinant esterase and use thereof |
Publications (3)
| Publication Number | Publication Date |
|---|---|
| WO2007073845A2 true WO2007073845A2 (en) | 2007-07-05 |
| WO2007073845A3 WO2007073845A3 (en) | 2007-08-02 |
| WO2007073845A8 WO2007073845A8 (en) | 2008-07-24 |
Family
ID=38017096
Family Applications (1)
| Application Number | Title | Priority Date | Filing Date |
|---|---|---|---|
| PCT/EP2006/011832 Ceased WO2007073845A2 (en) | 2005-12-27 | 2006-12-08 | Polypeptide having esterase activity and recombinant esterase and use thereof |
Country Status (14)
| Country | Link |
|---|---|
| US (2) | US8158393B2 (en) |
| EP (1) | EP1966373B1 (en) |
| JP (1) | JP5119166B2 (en) |
| KR (1) | KR101388391B1 (en) |
| CN (1) | CN101351548B (en) |
| AT (2) | AT502990A1 (en) |
| BR (1) | BRPI0621280A8 (en) |
| CA (1) | CA2635380C (en) |
| ES (1) | ES2383702T3 (en) |
| IL (1) | IL192400A (en) |
| NO (1) | NO343225B1 (en) |
| PL (1) | PL1966373T3 (en) |
| SG (1) | SG170757A1 (en) |
| WO (1) | WO2007073845A2 (en) |
Cited By (1)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| WO2010122175A1 (en) * | 2009-04-24 | 2010-10-28 | Dsm Ip Assets B.V. | Improved pig liver esterases |
Families Citing this family (1)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| PL2171061T3 (en) * | 2007-07-04 | 2019-03-29 | Patheon Austria Gmbh & Co Kg | Preparation of an esterase |
Citations (1)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| WO2002048322A2 (en) | 2000-12-12 | 2002-06-20 | Degussa Ag | Recombinant porcine liver esterases, their use and a method for the production thereof |
Family Cites Families (2)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| US5817490A (en) * | 1996-05-17 | 1998-10-06 | Eastman Chemical Company | Enzymatic process for the manufacture of ascorbic acid 2-keto-L-gulonic acid and esters of 2-keto-L-gulonic acid |
| DE10258327A1 (en) * | 2002-12-13 | 2004-06-24 | Degussa Ag | New artificial esterase, useful e.g. in washing compositions and for enantioselective reaction or hydrolysis of carboxylic acid derivatives, comprises that it is derived from porcine liver esterase by site-specific mutation |
-
2005
- 2005-12-27 AT AT0208105A patent/AT502990A1/en not_active Application Discontinuation
-
2006
- 2006-12-08 EP EP06829433A patent/EP1966373B1/en not_active Not-in-force
- 2006-12-08 CN CN200680049665.5A patent/CN101351548B/en not_active Expired - Fee Related
- 2006-12-08 PL PL06829433T patent/PL1966373T3/en unknown
- 2006-12-08 AT AT06829433T patent/ATE549400T1/en active
- 2006-12-08 BR BRPI0621280A patent/BRPI0621280A8/en not_active Application Discontinuation
- 2006-12-08 SG SG201102064-1A patent/SG170757A1/en unknown
- 2006-12-08 US US12/159,547 patent/US8158393B2/en not_active Expired - Fee Related
- 2006-12-08 ES ES06829433T patent/ES2383702T3/en active Active
- 2006-12-08 KR KR1020087018341A patent/KR101388391B1/en not_active Expired - Fee Related
- 2006-12-08 WO PCT/EP2006/011832 patent/WO2007073845A2/en not_active Ceased
- 2006-12-08 CA CA2635380A patent/CA2635380C/en active Active
- 2006-12-08 JP JP2008547868A patent/JP5119166B2/en not_active Expired - Fee Related
-
2008
- 2008-06-23 IL IL192400A patent/IL192400A/en active IP Right Grant
- 2008-06-27 NO NO20082864A patent/NO343225B1/en not_active IP Right Cessation
-
2012
- 2012-03-12 US US13/417,734 patent/US8642312B2/en not_active Expired - Fee Related
Patent Citations (1)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| WO2002048322A2 (en) | 2000-12-12 | 2002-06-20 | Degussa Ag | Recombinant porcine liver esterases, their use and a method for the production thereof |
Non-Patent Citations (1)
| Title |
|---|
| FEBS LETT., vol. 293, 1991, pages 37 - 41 |
Cited By (2)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| WO2010122175A1 (en) * | 2009-04-24 | 2010-10-28 | Dsm Ip Assets B.V. | Improved pig liver esterases |
| US8921080B2 (en) | 2009-04-24 | 2014-12-30 | Dsm Ip Assets B.V. | Pig liver esterases |
Also Published As
| Publication number | Publication date |
|---|---|
| SG170757A1 (en) | 2011-05-30 |
| EP1966373B1 (en) | 2012-03-14 |
| WO2007073845A8 (en) | 2008-07-24 |
| CA2635380A1 (en) | 2007-07-05 |
| IL192400A (en) | 2013-06-27 |
| ES2383702T3 (en) | 2012-06-25 |
| US20100151541A1 (en) | 2010-06-17 |
| BRPI0621280A8 (en) | 2017-09-19 |
| KR101388391B1 (en) | 2014-04-22 |
| IL192400A0 (en) | 2009-02-11 |
| KR20080093109A (en) | 2008-10-20 |
| NO343225B1 (en) | 2018-12-10 |
| EP1966373A2 (en) | 2008-09-10 |
| US8642312B2 (en) | 2014-02-04 |
| NO20082864L (en) | 2008-09-25 |
| AT502990A1 (en) | 2007-07-15 |
| CA2635380C (en) | 2014-10-21 |
| CN101351548B (en) | 2015-08-19 |
| CN101351548A (en) | 2009-01-21 |
| BRPI0621280A2 (en) | 2011-12-06 |
| US20120220014A1 (en) | 2012-08-30 |
| HK1128306A1 (en) | 2009-10-23 |
| ATE549400T1 (en) | 2012-03-15 |
| US8158393B2 (en) | 2012-04-17 |
| JP5119166B2 (en) | 2013-01-16 |
| JP2009521239A (en) | 2009-06-04 |
| PL1966373T3 (en) | 2012-08-31 |
| WO2007073845A3 (en) | 2007-08-02 |
Similar Documents
| Publication | Publication Date | Title |
|---|---|---|
| AU2003221082B2 (en) | Novel carbonyl reductase, gene encoding it and process for producing optically active alcohols using the same | |
| US8642312B2 (en) | Polypeptide having esterase activity and recombinant esterase and use thereof | |
| DK2013336T3 (en) | New group of esterases for the production of fine and specialty chemicals | |
| CN101641437B (en) | Isoforms of pig liver esterase | |
| US7229817B2 (en) | Recombinant porcine liver esterases, their use and a method for the production thereof | |
| AU2001284047B2 (en) | Butinol I esterase | |
| JP2003502021A (en) | Epoxide hydrolase of Aspergillus origin | |
| WO2007073847A1 (en) | Novel polypeptide having esterase activity and recombinant esterase and use thereof | |
| Simatupang et al. | Lipolytic activity of Itb1. 1 and Lk3 thermostable lipases expressed in Escherichia coli and Pichia pastoris | |
| JP2009521239A5 (en) | ||
| WO2007073846A1 (en) | Method for preparing enantiomerically enriched 2-alkyl-5-halopent-4-enecarboxylic acids and -carboxylic esters | |
| HK1128306B (en) | Polypeptide having esterase activity and ecombinant esterase and use thereof | |
| KR102884132B1 (en) | Lipases with equal stereoselectivity for sn-1 and sn-3 | |
| JP2001238682A (en) | Gene encoding reductase | |
| JPH03210183A (en) | Cloning, expression and sequence determination of esterhydrolase gene in colon bacillus |
Legal Events
| Date | Code | Title | Description |
|---|---|---|---|
| WWE | Wipo information: entry into national phase |
Ref document number: 200680049665.5 Country of ref document: CN |
|
| WWE | Wipo information: entry into national phase |
Ref document number: 2006829433 Country of ref document: EP |
|
| WWE | Wipo information: entry into national phase |
Ref document number: 2635380 Country of ref document: CA |
|
| WWE | Wipo information: entry into national phase |
Ref document number: MX/a/2008/008501 Country of ref document: MX Ref document number: 2008547868 Country of ref document: JP Ref document number: 5611/DELNP/2008 Country of ref document: IN |
|
| NENP | Non-entry into the national phase |
Ref country code: DE |
|
| WWE | Wipo information: entry into national phase |
Ref document number: 1020087018341 Country of ref document: KR |
|
| WWP | Wipo information: published in national office |
Ref document number: 2006829433 Country of ref document: EP |
|
| WWE | Wipo information: entry into national phase |
Ref document number: 12159547 Country of ref document: US |
|
| ENP | Entry into the national phase |
Ref document number: PI0621280 Country of ref document: BR Kind code of ref document: A2 Effective date: 20080627 |